Abstract
Global agricultural challenges, especially soil degradation caused by abiotic stresses, significantly reduce crop productivity and require innovative solutions. Biochar (BC), a biodegradable product derived from agricultural and forestry residues, has been proven to significantly enhance soil quality. Although its benefits for improving soil properties are well-documented, the potential of BC to mitigate various abiotic stresses-such as drought, salinity, and heavy metal toxicity-and its effect on plant traits need further exploration. This review aims to elucidate BC production by highlighting primary feedstock’s and synthesis techniques, and examining its role in boosting soil decomposition efficiency and fertility, which are pivotal for sustainable crop growth. This review also discuss how BC can enhance the nutritional and chemical properties of soil under different abiotic stress conditions, emphasizing its capacity to foster crop growth and development in adverse environments. Furthermore, this article serves as a comprehensive resource for agricultural researchers in understanding the importance of BC in promoting sustainable agriculture, and addressing environmental challenges. Ultimately, this review highlights critical knowledge gaps and proposes future research avenues on the bio-protective properties of BC against various abiotic stresses, paving the way for the commercialization of BC applications on a large scale with cutting-edge technologies.
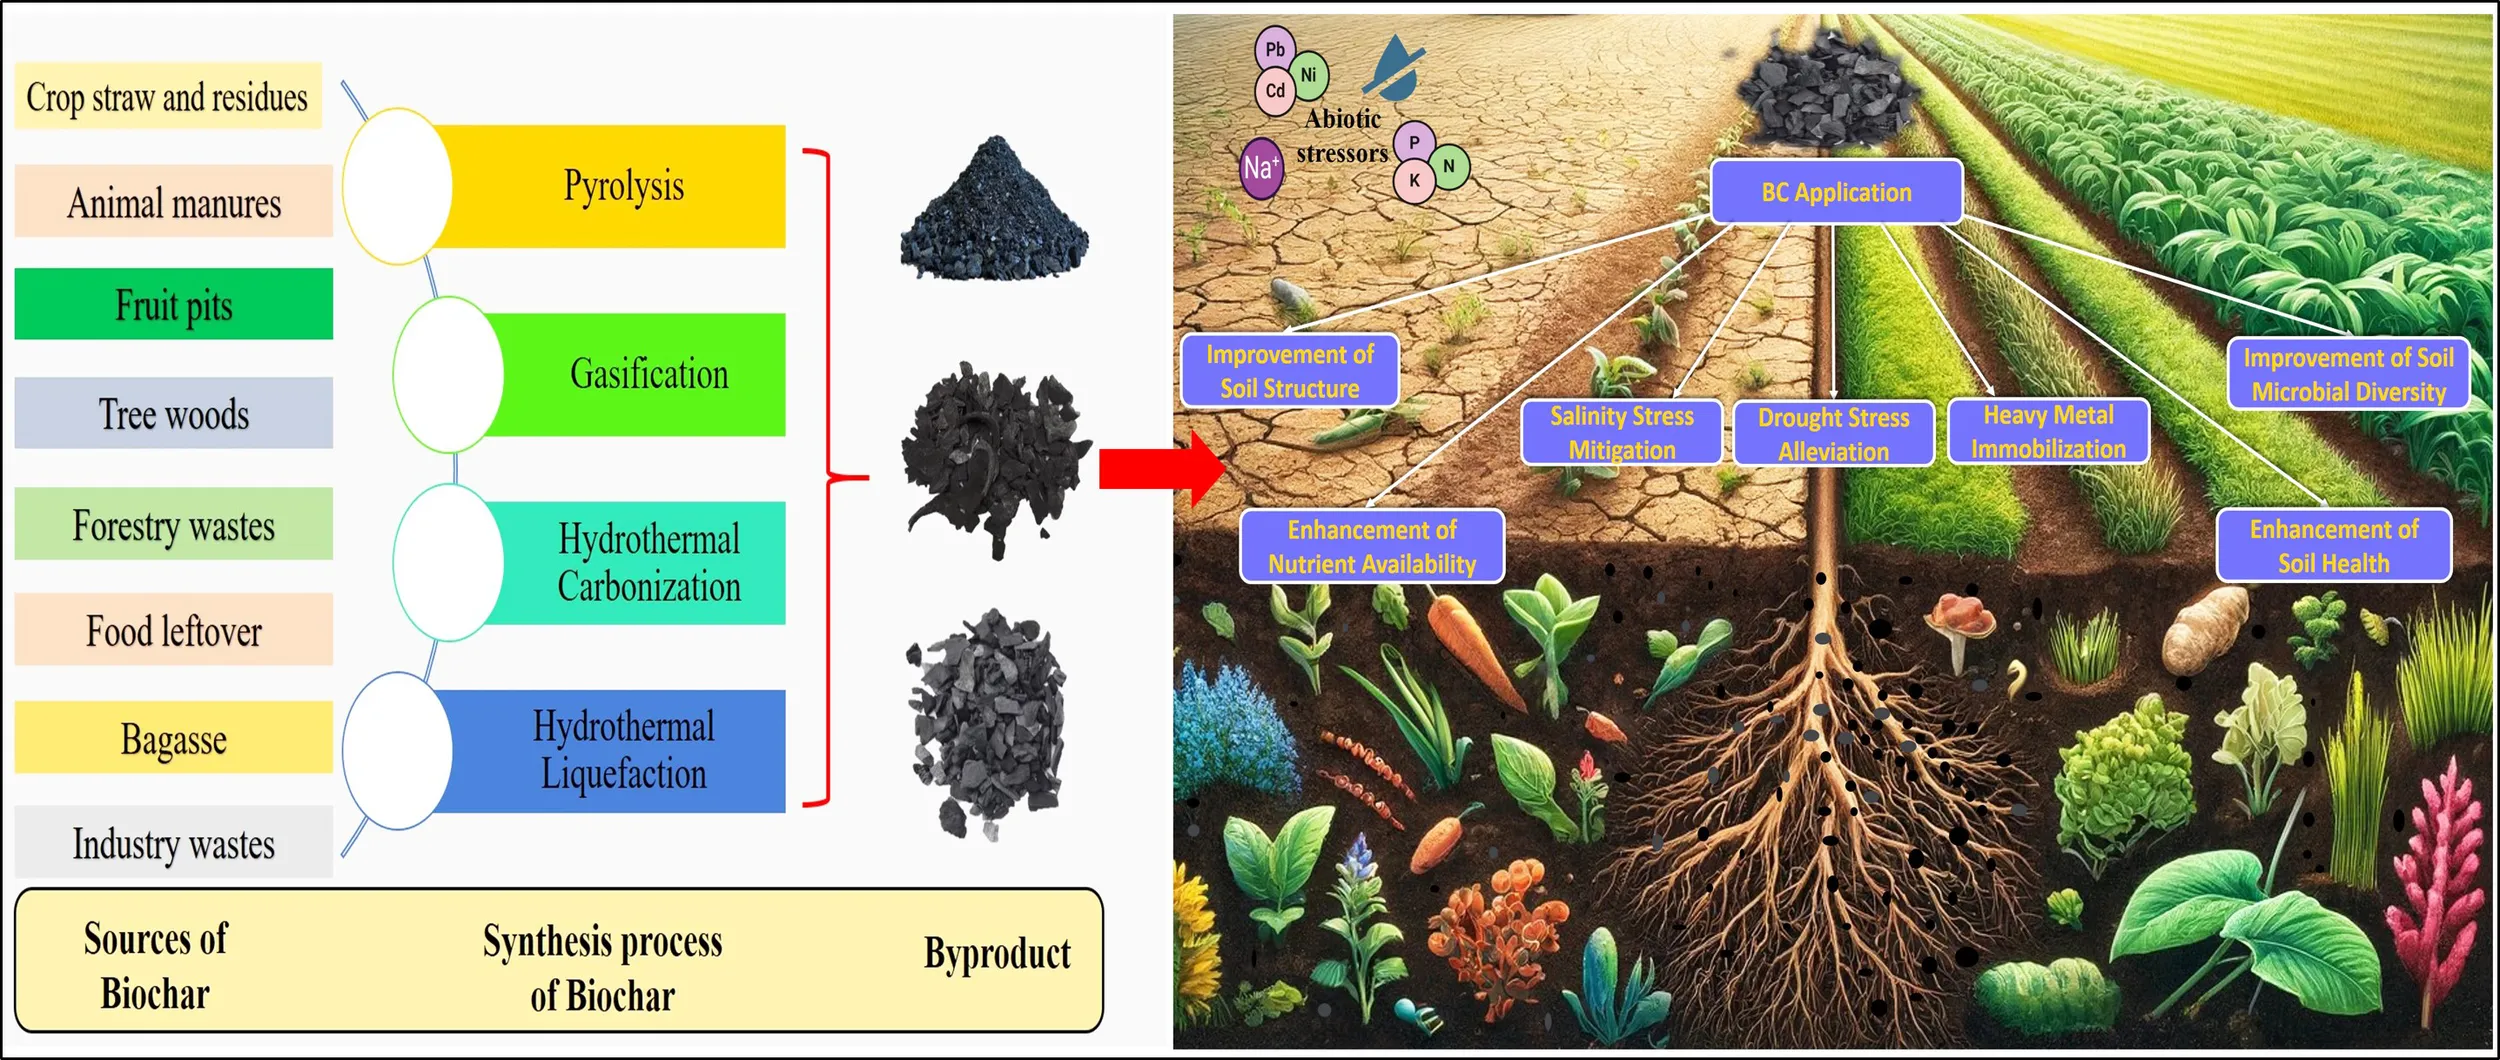
Highlights
BC ameliorates physico-chemical properties of soil against environmental stress.
It serves as a significant nutritional reservoir for plant growth improvement.
BC acts as a key player in mitigating abiotic stress tolerance for sustainable agriculture.
Further studies are needed on expression pattern and characterization of genes in BC’s protective roles against abiotic stress.
Emphasis should be placed on innovative uses of BC for agricultural stress management.
1 Introduction
Soil degradation, severe soil contamination and loss of soil fertility provoke a global threat to food security and agricultural sustainability. Rising food deficits and climate change need a green solution for improving soil quality and diminishing ecological agriculture impacts to ameliorate crop productivity. The excessive use of chemical fertilizers with salt and other acidic components reduces the productivity of crops by triggering soil quality via soil deterioration, soil acidity, and poor soil aggregate structures (Wu et al., 2023). Quality of soil is commonly affected by soil organic matter (OM), electrical conductivity (EC), and soil depth, which cause salinization, compaction, nutrient deficiency, erosion, loss of biodiversity and desertification, which all lead to soil fertility reduction (; Lal, 2015). In addition, soil nutrient depletion was directly associated with food insecurity due to unsustainable land use. To combat this, various soil additives are implemented to augment soil nutrients, including composts, inorganic chemical fertilizers, seaweed, organic manures, mulches, clay minerals, nanomaterials and sewage sludge, etc (; Yasmeen et al., 2022). Since most of these management approaches have less or no impact on the storage of soil carbon (C), prompt organic C (OC) decomposition results in the emission of carbon-di-oxide (CO2), thereby reducing the efficiency of C balance (; ). Hence, sustainable and reliable resource management techniques are urgently needed to mitigate global soil contamination and restore soil quality (Pradhan et al., 2018).
Global agricultural productivity has been significantly impacted by various abiotic stressors, which are major limiting factors affecting soil quality. Abiotic stressors such as drought, soil salinity, and heavy metal accumulation contribute to over 50% of crop production losses and affect 91% of the world’s cropland (Younis et al., 2020). Among these, heavy metal pollution, a notable consequence of anthropogenic activities, has significantly increased since the industrial revolution. For instance, high concentrations of heavy metals in soils adversely affect plant physiology, metabolism, and biochemical processes, leading to reduced growth, biomass, and yield of plants (Goyal et al., 2020). In addition to heavy metal pollution, reduced precipitation due to climate change has exacerbated global drought conditions. Drought stress reduces cell turgor and negatively impacts plant growth. It reduces shoot growth, limiting the production and transfer of photosynthetic materials, which ultimately decreases plant growth and yield (Nour et al., 2024). For example, severe drought stress reduced yield of rice (Oryza sativa) (53-92%), wheat (Triticum aestivum) (57%), maize (Zea mays) (63-87%), soybean (Glycine max) (46-71%) and chickpea (Cicer arietinum) (45-69%) (). Similarly, salinity stress reduces crop yield, with declines ranging from 5-50% due to osmotic stress, ionic toxicity, and nutrient imbalances (Okorogbona et al., 2015).
To meet the projected increase in food demand for an estimated global population of 9 to 10 billion people by 2050 (Van Dijk et al., 2021), various strategies have been implemented to improve crop performance under abiotic stress. These strategies include breeding techniques, agronomic practices, seed priming, microbial seed treatment, microorganism inoculation, grafting, and the use of plant growth regulators and osmoprotectants (Gupta and Shrestha, 2023; Oyebamiji et al., 2024). Especially, farmers use pesticides and hazardous chemical fertilizers to cultivate maximum crops in a minimal area, which further lowers land quality and causes soil degradation, contamination, erosion and water pollution (; Oliver and Gregory, 2015; Pradhan et al., 2018). To combat this, the application of biochar (BC) has recently emerged as a cost-effective and environment friendly strategy to enhance crop tolerance to abiotic stress.
BC is a highly stable carbonaceous residue resulting from the thermochemical degradation of various feedstocks, such as crop residues, mill residues, agricultural wastes, food wastes, animal manure, and forestry wastes (Tomczyk et al., 2020). BC is valued for its micro-pores and high cation exchange capacity (CEC), which do not exacerbate environmental conditions. It is primarily composed of oxygen (O2), nitrogen (N), hydrogen (H), C, and aromatic and alkyl matter (Nath et al., 2022). BC’s unique structural and functional properties make it a valuable soil amendment for enhancing soil fertility. In USA and China alone, approximately 1.4 BT of agro-biomass waste are generated annually, producing around 420 MT of BC per year (Godlewska et al., 2017; Nath et al., 2022; Kumar et al., 2023). BC has been shown to enhance crop growth and yield under abiotic stresses and in metal-polluted soils. Incorporating BC into infertile or nutrient-deficient soils can improve crop performance, benefit farmers, reduce the use of inorganic fertilizers, and support environmental conservation (; Wani et al., 2022). Raw BC has a limited ability to absorb contaminants from highly polluted water (Jagadeesh and Sundaram, 2023). Furthermore, the small particle size of powdered BC makes it difficult to separate pollutants from the contaminated water (Sivaranjanee et al., 2024). Nowadays, several studies focus on synthesizing novel BCs using nanocomposites to remove aqueous contaminants in an effort to overcome these unfavorable factors (Li et al., 2023; ). This type of nanocomposite-based BC method helps to improve the physical and chemical properties of BC. For instance, the nanocomposite BC exhibits higher porosity, more surface active sites, increased stability, a larger specific surface area, and a wider range of applications compared to the unaltered BC (Pan et al., 2021). Various review articles have well described the synthesis of BC nanocomposites (; ; Lalhriatpuia and Tiwari, 2023). Hence, we can use this type of BC to remove heavy metal pollutants from wastewater and support efforts to improve the aquatic environment. To date, there is no much comprehensive review on the role of BC in alleviating abiotic stresses in plants. This review aims to highlight the production of BC from crop residual biomass and its wide range of applications under abiotic stress conditions. In addition, it provides updated information on BC for improving soil fertility and crop growth. Furthermore, we have discussed what studies should be carried out to understand the exact role of BC in crop development against abiotic stresses. Overall, we believe this review enhances the understanding of the role of crop residue-derived BC in controlling hazardous chemical-based soil amendments, reducing anthropogenic gas emissions, and ensuring environmental sustainability. Apart from this, this review will raise awareness in plant molecular biology researchers to initiate in depth molecular experiments to study about gene regulations on using BC for plant growth.
2 Methodology
Published research articles related to the topic were collected from five scientific databases, including Web of Science, “Scopus,” “PubMed,” “Science Direct,” and “Google Scholar”. The following combinations of search terms were used to collect articles: “role of BC on improving soil properties,” “biochar role in physical and chemical properties of soil,” “BC synthesis methods,” “Effects of biochar on drought stress tolerance in plants,” “Effects of biochar on salinity stress tolerance in plants,” “Effects of biochar on heavy metal stress tolerance in plants,” and “Role of biochar for improving abiotic stress tolerance in plants.” This review included articles published in English up until August 2024. Article titles and abstracts were manually assessed to exclude reports that were not relevant to this review. This review includes only biochar-related topics that enhance abiotic stress tolerance. We excluded only articles published in languages other than English.
3 Feedstock for BC synthesis
Effective selection of feedstock biomass is crucial for optimizing the preparation and yield of BC. Biomass feedstock, a complex solid material, can be categorized as either woody or non-woody. The classification of biomass applied for BC production is mainly based on its source, biological diversity and origin. Plant biomass and organic waste are the two main sources of feedstock used for BC production. In organic waste feedstocks, the use of various types of crop residue biomass for BC production has gained attention due to its economic benefits, environmental advantages, and scientific interest (). Crop residue biomass includes materials that are not classified as processed or field residues, such as leaves, straw, stalks, shells, molasses, roots, husks, peels, bagasse, tree prunes, and pods, sourced from agricultural lands, homes, and industries.
Straws, for instance, can be converted into bioplastics, chemicals, biogases, enzymes, and biocatalysts (). Global estimates indicate that rice straw production is around 800-1000 MT, while wheat straw production is approximately 354 MT, consisting of cellulose (32-47%), lignin (5-24%), and hemicellulose (19-27%) (; Ingrao et al., 2021).
Bagasse, a multicellular lignocellulosic residual fiber extracted from sugarcane and other sources such as pomegranate, pineapple, cashew, and sorghum, is another significant biomass. In 2021, the production of sugarcane reached 1.6 BT, generating 279 MMT of sugarcane bagasse. Bagasse has numerous applications, including biofuel, ceramics, cement additives, bricks, catalysts, concrete, adsorbents, food additives, silage feed, and organic manure ().
Pruned branches from fruit trees like apples, pears, and plums are abundant sources of lignocellulosic biomass. Farmers often incinerate these branches to reduce insect pests and plant diseases, contributing to atmospheric CO2 emissions (Sasaki et al., 2014). In 2010-2011, 1650 tons of pruned pear branches were reported to be discarded and accumulated in fields by the Tokushima Agriculture, Forestry, and Fisheries Technology Support Center of the Fruit Tree Research Institute (Sasaki et al., 2014). Utilizing pruned branches holds potential for BC and biofuel production.
The characteristics of BC derived from diverse crop residues have been compared in numerous studies (Wu et al., 2012; Windeatt et al., 2014; Purakayastha et al., 2015). For instance, Purakayastha et al. (2015) prepared four types of BC from maize stover, pearl millet stalk, rice straw, and wheat straw, finding that maize BC had higher nutrient values, particularly N and phosphorus (P), and greater C stability compared to other crop-derived BC. The study also determined that the total C content was highest in maize BC (66%), followed by pearl millet BC (64%), wheat BC (64%), and rice BC (60%). Another study utilized eight different crop-derived feedstocks, including coconut husk, coconut shell, cotton stalk, olive pomace, palm shell, rice husk, sugarcane bagasse, and wheat straw, for BC production, yielding 28% to 39% of BC. This study also found that high lignin feedstocks produced high-C BC with significant recalcitrance (Windeatt et al., 2014). Wu et al. (2012) demonstrated that rice straw-derived BC had high alkalinity, CEC, and levels of available P and extractable cations, indicating its potential as a fertilizer and soil amendment. Comparative analysis of BC production from various crop residue feedstocks is still limited, and it is necessary to identify the most suitable feedstocks for high-value BC production on a large scale.
While specific data on the annual production of crop residues are unavailable, recent statistics (FAO, 2022; MMR, 2023) indicate that the global cultivation of primary crops increased by 52%, fruits by 55%, and vegetables by 65% between 2000 and 2020 (Figure 1). This significant increase suggests a corresponding rise in crop residue production each year. Converting these residues into BC is a vital sustainable waste management strategy that mitigates climate change, enhances plant growth, and protects the environment.
Figure 1
4 BC synthesis methods
BC can be synthesized through various thermochemical techniques, mainly pyrolysis, gasification, hydrothermal carbonization (HTC), and hydrothermal liquefaction (HTL). The production conditions and physico-chemical properties of used biomass resources for BC synthesis play a vital role in porosity, CEC, specific surface area, functional groups and yield percentage (Nath et al., 2022; Singh et al., 2022). Table 1 presents the different techniques used for BC synthesis.
Table 1
| Synthesis technique | Description | Advantages | Reference | |
|---|---|---|---|---|
| Traditional approach | Firebrick pits, clay heater, iron and brick retort furnace are used as a reactors and feedstock burnt directly in an open field covered partially with half burned biomass or soil to reduce oxygen supply | Low cost No energy consumed Advanced technical skills are not required | Thines et al., 2017; Gabhane et al., 2020; Masek, 2022 | |
| Conventional pyrolysis | Slow | TR: 300-600 °C; HR: 5-7 °C; min-1 RT: 60-120 min O2 supply: Nil | Energy consumption was less Moderate TR | Mendez et al., 2015; |
| Fast | TR: >500 °C; HR: 300 °C; min-1 RT: 0-20 min O2 supply: Nil | Conversion rate higher Low RT Better yield Higher amount of bio-oil produced Large-scale BC synthesis | Mendez et al., 2015; Laird et al., 2017 | |
| Flash | TR: >1000 °C; HR: 1000 °C; sec-1 RT: 0-1 min O2 supply: Nil | Fast, effective, and efficient technique | Gabhane et al., 2020; | |
| Gasification | TR: >700 °C; Gasifying agents: Air, steam, O2, and CO2 | Humid biomass was used Produced high quality BC, C2H4, C2H2, other useful fuels and eco-friendly chemicals Efficacious environmental, and economic benefits | You et al., 2018; ; Zhang et al., 2022 | |
| HTC | TR: 150-350 °C; Pressure: 2-10 MPa RT: Several hours O2 supply: Less or Nil | Biomass predrying not required Wet biomass can be directly converted into byproducts Enhanced hydrophobicity or dewater ability of feedstock | Pauline and Joseph, 2020; ; Moreira et al., 2021 | |
| HTL | TR: 250-374 °C; Pressure: 2-25 MPa | No predrying of feedstock required Recovers <70% as bio-oil and BC Less water usage | Gollakota et al., 2018; | |
Details of BC production techniques and advantages.
TR, temperature range; HR, heating rate; RT, residence time; HTC, hydrothermal carbonization; HTL, hydrothermal liquefaction.
4.1 Pyrolysis process
Pyrolysis is an ancient method frequently used for synthesizing BC from biomass in chemical or thermal conversion methods. Pyrolysis is the thermal decomposition of biomass under elevated thermal vibration. During pyrolysis or incineration with a low O2 supply, crop residue breaks down organic components into condensable liquids, noncondensable gases, and char (Jung et al., 2019). Generally, pyrolysis products are composed of flammable methane (CH4), ethane (C2H6), H2, and (carbon monoxide) CO syngas, and liquid products are composed of phenolics, furanics, fatty acids, fine chemicals, biofuels, and solid material of BC (Fahmy et al., 2020; Wang et al., 2020a; ). In accordance with the TR, HR and, RT, conventional pyrolysis can be classified as slow, fast, ultrafast, or flash pyrolysis. In slow pyrolysis, the ranges of HR 5-7 °C; min-1, RT 60-120 min and TR 300-600 °C; can predominantly yield 20-30% syngas, 25-35% bio-oil and 35-45% BC, respectively. Fast pyrolysis occurs without O2 at HR 300 °C; min-1, RT 0-20 min, TR >500 °C; and synthesis 20% of syngas, 60% of bio-oil and 20% of BC. Ultrafast or flash pyrolysis carried out in a fluidized bed reactor with HR ≥1000°C sec-1, RT ≤1 min, TR ≥1000°C yields solid 10-15%, liquid 70-80%, and gas 5-20%. This ultrafast pyrolysis limits wide industrial application since it produces high bio-oil but low levels of BC (Laird et al., 2017; ; ).
The BC yield during the pyrolysis process depends on the type and nature of biomass used. Temperature is the main operating process condition that decides the product efficiency. Generally, the yield of BC decreases and the production of syngas increases when the temperature is increased during the pyrolysis process. For instance, study illustrated that the molecular properties and Cu sorption capacity of BC, derived from Jerusalem artichoke stalks, are closely related to the temperature of pyrolysis (Wei et al., 2019). In that study, the content of O2-containing functional groups in the BC samples decreased, while that of aromatic structures and alkaline mineral components increased, with a rise in pyrolysis temperature (Wei et al., 2019). However, Sawargaonkar et al. (2024) confirmed that peanut shell BC obtained through slow pyrolysis process has greater BC yield as compared to the fast pyrolysis, irrespective of reaction temperature, thus it confirms the effectiveness of the slow pyrolysis mechanism toward the BC production. Wan et al. (2014) compared the characterization of BC derived from rice husk and elm sawdust by fast pyrolysis. They demonstrated that high in ash, while low in volatile and fixed C content found in rice husk derived BC compared to elm sawdust derived BC. This study represents the characteristics of BC was mostly determined by sources of feedstock rather than synthesis process. In general, BC sizes were varied in the range <150 to 2000 µm in pyrolysis process (Liu et al., 2017a; ).
4.2 Gasification
Gasification is an effective waste management process comprising steps like drying, pyrolysis, combustion, and partial oxidation (You et al., 2018; Siwal et al., 2020; ). During gasification, partial oxidation enriches the chemical and textural properties of BC (Yaashikaa et al., 2020). At temperatures ranging from 700-1500°C, the heating rate is rapid, and the reaction duration varies from seconds to minutes, yielding ˜ 85% gas, 10% liquid, and 5% solid (). Depending on availability, air, steam, CO2, O2, and their mixtures used in gasification, significantly enhance BC’s physico-chemical properties, biomass conversion efficiency, product composition, and gas synthesis (You et al., 2018; Maya et al., 2021).
Generally, the BC yield from gasification is lower than that from pyrolysis, this was attributed to C conversion to CO under partial oxidation conditions. Additionally, gasification BC has smaller specific surface areas and total pore volumes compared to slow and fast pyrolysis BC, mainly due to ash melting (pore clogging), pore expansion and collapse, and tar deposition at high combustion and reduction temperatures. However, previous study indicated that higher temperatures and varied gaseous conditions in gasification led to lower BC yields but larger total surface area, higher pH and ash contents, and very low tar content (16-polycyclic aromatic hydrocarbons) (Fryda and Visser, 2015). The particle sizes of gasification BC ranged from under 45 μm to over 2000 μm, showing inconsistency across studies (Griffith et al., 2013; Pujol Pereira et al., 2016; Shen et al., 2016).
4.3 Hydrothermal carbonization
HTC is a highly effective method for converting wet biomass into valuable byproducts without the need for pre-drying. The process operates within a reactor under pressures of 2-10 megapascal (MPa) and temperatures ranging from 150-350 °C;, with minimal or no O2 present, and lasts for several hours. The HTC process involves hydrolysis, dehydration, decarboxylation, aromatization, and re-condensation, producing syngas, hydro-char, and bio-oil (; ).
Similar to pyrolysis, HTC generates a solid product of BC (called hydro-char), which makes up to 50-80%, along with a bio-oil and water mixture (5-20%), and CO2 (2-5%) (Saqib et al., 2019). However, hydro-char produced via HTC typically not classified as BC due to insufficient reaction temperatures, low C content, and an unfavorable O/C and H/C ratio (Wiedner et al., 2013). Recent research shows that combining HTC with pyrolysis can enhance BC quality and stabilize heavy metals in the final solid product (Li et al., 2022a). Olszewski et al. (2019) found that pre-treating brewery spent grains with HTC before pyrolysis significantly improves BC yield and C content, while reducing ash composition. Garlapalli et al. (2016) also observed an increase in C content to 82% in BC produced from the combined HTC and pyrolysis process, compared to 70% from HTC alone. Overall, improving hydro-char is crucial due to its low surface area (<30 m²/g), poor porosity, and the presence of harmful chemicals like furan, furfural, and phenolic compounds, which limit its use in soil improvement applications.
4.4 Hydrothermal liquefaction
In HTL, macro algae and lignocellulosic feedstock are broken down under high pressure and temperature in supercritical or critical water conditions to produce bio-oil, solids, gases, and organic byproducts. This process operates in a water medium at temperatures between 250-374 °C; and pressures of 5-20 MPa. HTL reactions involve the depolymerization of macromolecules, thermal decomposition, and recombination processes (Mathanker et al., 2021; Gollakota et al., 2018). The decomposition phase includes dehydration, decarboxylation, and deamination of the biomass, generating furfurals, phenols, soluble organic acids, polar organic molecules, and glycolaldehydes. Repolymerization and recombination are reverse processes of depolymerization, occurring upon the loss of H2 ions which act as free radicals. In the absence of H2, previously synthesized compounds repolymerize to form coke, a robust molecular complex (Ni et al., 2022; Ravichandran et al., 2022). HTL achieves a recovery of less than 70% of its feedstock as bio-oil and BC.
The high BC yield in HTL is estimated up to 70%, but have some challenges since biomass polymers are less likely to be converted to solid phases under hydrothermal conditions compared to other thermochemical processes like pyrolysis. Research indicates that the surface area and total volume of HTL BC are generally lower than those of pyrolysis BC, regardless of the feedstock used (Guo and Rockstraw, 2007; Leng et al., 2015). The surface area ranges from 1.56 to 17 m²/g, the average pore diameter from 18 to 36 nm, and the total pore volume from 0.058 to 0.082 cm³/g (Kumar and Pant, 2015; Leng et al., 2015). Despite these differences, HTL BC retains functional groups and volatile organic matter crucial for the adsorption of metals, dyes, and other pollutants. While HTL demonstrates efficient performance, economic viability, and a high production rate, it still faces numerous operational and technical challenges that hinder its full commercialization.
Most of the above-discussed biomass-derived BC synthesis processes are less expensive, more convenient and farmer-friendly approaches than typical activation methods. A schematic representation of various BC synthesis methods can be seen in Figure 2.
Figure 2
5 Influence of BC physico-chemical soil properties
Improving soil health and adopting sustainable practices will boost crop yields, ensuring food security and environmental sustainability for the future. The impact of BC on soil properties has been widely studied. Morphological characteristics (e.g., large surface area and highly porous structure) of BC can change soil physical and chemical properties, which have been linked to changes in soil microbial community.
5.1 Impact of BC on physical properties of soil
Using BC as a soil amendment significantly increased various physical properties of soil such as BD, TP and WA.
5.1.1 Soil bulk density and total porosity
The application of BC has been shown to significantly reduce BD and increase TP by indirectly influencing soil aggregation (Li et al., 2024). This process begins with a reduction in BD, followed by enhanced soil aggregation, interaction with mineral soil particles, and ultimately decreased soil packing. Lower BD can enhance soil structure, improve nutrient release and retention, and reduce soil compaction. Similarly, higher TP provides essential space and oxygen for soil organisms, influencing the transformation, storage, and utilization of water.
Studies have indicated that BC amendment improves BD, agglomerate stability, and aggregate capacity, thereby enhancing water retention and preventing soil degradation (Wang et al., 2020b). Consistent with Zhang et al. (2012a, 2012b), the addition of 40 t ha-1 rice straw BC to the soil reduced BD from 0.1 to 0.06 g cm-3 in 2009 and 2010, while increasing rice yield by 9-12% and 9-28%, respectively. Changes in TP were observed in the 5–10 and 25 μM ranges following BC addition (Rasa et al., 2018). Furthermore, BC implementation significantly enhanced soil permeability and saturated hydraulic conductivity (Oguntunde et al., 2008).
Jeffery et al. (2011) found that BC supplements significantly enhanced crop productivity in soils with acidic pH (14%), neutral pH (13%), and coarse (10%) or medium textures (13%). Sun and Lu (2014) found that straw bulk BC significantly increased pore volume in the macropore (> 75 μm) and mesopore (30-75 μm) ranges, likely due to the reorganization of pore-size distribution and aggregation processes induced by BC addition.
Overall, the impact of BC on BD and TP is closely related to the type of BC, soil type, BC particle size, and application rate. For example, Verheijen et al. (2019) demonstrated that smaller BC particles more effectively reduced the BD of sandy soil, while larger BC particles had a greater effect on reducing the BD of sandy loam soil, indicating that various BC particle sizes can be used to achieve specific soil effects. Similarly Rasa et al. (2018) highlighted that BC chemistry and pore morphology influence BC-water interactions, thereby altering soil textures accordingly.
5.1.2 Water availability
Studies have demonstrated that BC significantly enhances WA in both sandy and clay soils (Ma et al., 2016; Pu et al., 2019). This is attributed to the porous nature of BC, which allows it to absorb substantial amounts of water, thereby altering the overall soil structure. In sandy soils, incorporating BC particles of various sizes and shapes can reduce the large gaps between soil particles (interpore spaces) and increase the proportion of micropores (5 to 30 µM in diameter) formed by the intrapores of BC. Consequently, when BC-sand mixtures become moist, the elongated shape of BC particles disrupts the grain packing in the sandy matrix, enhancing the interpore volume available for water storage (Liu et al., 2017b; Lehmann and Joseph, 2024). Applying BC at rates exceeding 3% w/w has been shown to potentially increase WA in clay soils (P < 0.05) (Kameyama et al., 2016). In a meta-analysis by Razzaghi et al. (2020) reported that BC additions increased available water content by 45% in coarse-, 21% in medium- and 14% in fine-textured soils. In clay soils, BC additions generally improve hydraulic conductivity and field capacity while reducing BD, thereby enhancing drainage, porosity, and plant-available water.
5.2 Impact of BC on chemical properties of soil
Soil chemical properties such as available N, P, potassium (K), pH, soil electrical conductivity was highly influenced by BC application.
5.2.1 Nutrient availability
The soil environment is crucial for plant growth, and BC manifestation for long time showed to enhance soil nutrient availability and improve plants’ nutrient absorption efficiency. Therefore, BC can also be utilized as a vital nutrient source for plants and soil microorganisms. The higher levels of K, N, calcium (Ca), and P available in BC render nutrients to microorganisms essential for plant growth (Sakhiya et al., 2020). Hossain et al. (2020) reported that OC and essential minerals such as Ca, K, P, N, sulfur (S), and magnesium (Mg) were elevated via BC treatment in the soil. Gao et al. (2016) found that an increased retention of NO3 N (33%) and NH4+ N (53%) has a more significant effect in the soil upon BC amendment than direct nutrient supplements. Furthermore, BC application resulted in an increased grain P (38-230%) and N (20-53%) utilization efficiency compared to N fertilizer alone (Zhang et al., 2020a).
5.2.2 Soil pH
BC application can also potentially modify common soil indicators such as pH, and electrical conductivity (Murtaza et al., 2023). Soil pH has a profound impact on plant growth and available nutrients. Generally, in agricultural fields, soil acidity (pH) increases through the application of lime to improve plant growth at maximum potential. The application of BC was found to rise the pH from 4.59 to 4.86 (Nielsen et al., 2018), from 4.8 to 6.3 (Novak et al., 2009), and from 4.3 to 4.6 (Hossain et al., 2010). Earlier studies showed that utilization of higher pH BC simultaneously increased pH in red ferralitic soil at approximately the 1/3 lime level, improved the Ca ratio and decreased Al toxicity (Glaser et al., 2002; Lehmann et al., 2003; Steiner et al., 2007). Granatstein et al. (2009) found that applying 39 t ha−1 herbaceous feedstock-derived BC to sandy soil increased the soil pH from 7.1-8.1. found a significant increase in 71% electrical conductivity and a 5.2-7.6 pH range in sandy soils treated umbrella tree-derived BC compared to untreated controls. Mostly, BC was reported to not have any effect on light and highly acidic soils (Sousa and Figueiredo, 2016). Whereas, BC significantly increase the pH value of highly acidic to light alkaline soils (; Wen et al., 2022). Moreover, some studies revealed that increasing temperature during pyrolysis process has contributed to increase in soil pH by BC (Wan et al., 2014; Karimi et al., 2020).
5.2.3 Cation exchange capacity and electrical conductivity
The CEC measures the soil’s ability to absorb, retain, and exchange cations. Enhancing the number of cation exchange sites in the soil can boost its CEC content. Soils with a high CEC are more capable of adsorbing NH4+, K+, Ca2+, and Mg2+, which enhances the efficient use of nutrient ions and minimizes nutrient loss (Liang et al., 2006). Higher CEC in soil supports plant nutrient cations binding to the clay, and humus to retain nutrients for uptake by plants instead of leaching (Glaser et al., 2002; Lehmann et al., 2003; Laird et al., 2010). After the addition of BC, the soil charge and CEC is reported to be increased by approximately 20–40% (Hossain et al., 2010). The anionic surface of BC was mainly attributed to increase the CEC of soil with both acidic and alkaline pH (). Tomczyk et al. (2020) found that woody BC enhanced the CEC of generated soil by 190% when compared with the untreated control. BC’s functional groups on the surface, silicon, alkalinity, and high pH-buffering capability contribute synergistically to moderate soil acidity (Mandal et al., 2020). The anion exchange capacity and CEC of the soil was also found to be emphasized by the incorporation of BC (Hossain et al., 2020).
5.3 Impact of BC on soil biological properties
The overall change of soil physical and chemical properties by the application of BC will result in the creation of appropriate habitat for living of beneficial microorganisms (Xu et al., 2014). In addition, due to the presence of high aromatic hydrocarbon and pore structure, BC served as a potential habitat and providing nutrient for various beneficial soil microorganism and resulted in improved crop productivity (). By increasing soil pH, BC renders the soil environment more beneficial for plant and microbes (). The micro and meso pores of BC stores water and dissolved substances required for the microbial metabolism. According to Li et al. (2022b), BC application has distinctive attributes, such as an altered strategy in root growth, enhanced enzyme activities and rhizosphere nutrient availability in soil. Plant growth regulators, karakins and other germination hormones released by BC trigger seed germination and soil physico-chemical properties (Kochanek et al., 2016). The efficacy of plant growth improvement with various BCs has been studied extensively (Table 2). The BC amendment augments soil microbial activity and diversity, which is fundamental for nutrient cycling, organic matter decomposition, and the overall health of the soil ecosystem (Hou et al., 2024). Microbial activity enhancement further aids in the stabilization of heavy metals and improves soil resilience to abiotic stresses (Pathy et al., 2020). Moreover, BC increases soil bacterial diversity and alter its structure (Huang et al., 2022).
Table 2
| Plant name | Botanical name | BC feedstock | Pyrolysis temperature | Level of BC | Effects of BC on plant growth enhancement | References |
|---|---|---|---|---|---|---|
| Pumpkin | Cucurbita pepo | Maize straw | 350 °C | 10 and 20 t ha−1 | Improved leaf RWC | Langeroodi et al., 2019 |
| Tomato | Lycopersicon esculentum | Cotton seed shell and rice husk | 400°C | 5% (w/w) | Increased RWC and leaf photosynthetic rate | |
| Apple | Malus domestica | Rice husk | 450 °C | 80 g k−1 | Increased seedling height, DW, respiration rate, higher root surface area, root length and root volume | Wang et al., 2019 |
| Asian lotus | Nelumbo nucifera Gaertn. | Pinewood | – | 10% (w/w) | Increased FW of leaf, root, DW of rhizome and relative Chl contents | Liu et al., 2016 |
| Chickpea | Cicer arietinum | Red sage | 450°C | 3.5 t ha-1 | Higher seed yield, haulm yield, and biological yield | Meena et al., 2023 |
| Sweet basil | Ocimum basilicum | Black cherry wood | 450°C | 2 and 3% (w/w) | Seed germination increased, improved Chl contents, enhanced surface area, total root volume and length | Jabborova et al., 2021a |
| Ginger | Zingiber officinale | Black cherry wood | 450°C | 1, 2 and 3% (w/w) | Increased seed germination, leaf length, leaf number, DW of shoot and root | Jabborova et al., 2021b |
| Peanut | Arachis hypogaea | Maize straw | 600°C | 10 and 20 t ha−1 | Photosynthesis, Chl fluorescence, and yield | Wang et al., 2021 |
| Tomato, Radish, Lettuce and Sweet pepper | Raphanus sativus, Lactuca sativa and Capsicum annuum | Maritime pine wood chips | 600°C | 2 kg/m2 = 10 t ha−1 | Increased mean FW and improved fruit and vegetable yield | Gonzalez-Pernas et al., 2022 |
| Maize | Zea mays | Hardwood | – | 18.4 Mg ha−1 | Highest grain yield and zero removal of residue | Rogovska et al., 2016 |
| Tea | Camellia sinensis | Tea plants | 550°C | 20 g | Higher macronutrient contents such as N, P, and K, enhanced the leaf biomass, stem biomass, and stem diameter | Zou et al., 2023 |
Ameliorative effects of various BCs on crop growth, development and yield.
RWC, relative water content; DW, dry weight; FW, fresh weight; Chl, chlorophyll.
5.4 Decomposition properties of soil
The chemical composition in feedstock obtained from different sources affects the biological decomposition of BC (Lehmann et al., 2011). The decomposition rate was significantly higher (mean: 0.025% day 1) in crop-derived BC than (mean: 0.007% day 1) grass-derived BC as a result of lower condensed and less C content. Furthermore, wood-derived BC (mean: 0.004% day 1) contains the lowest decomposition rate due to its high C content (Hilscher et al., 2009; Knicker, 2010; Singh and Cowie, 2014). Wang et al. (2016) found that BC decomposition rates increased logarithmically over time and were significantly influenced by soil texture, clay content, biomass feedstock, pyrolysis temperature, and process duration. Limited information is known about BC degradation, and the effects on the turnover of native soil organic matter, degradation duration and other cascading effects remain unclear (Lehmann et al., 2011; ; Lorenz and Lal, 2014). Previously, the application of BC in different soils has been reviewed; however, an updated overview of the persistence, degradation, and stability of BC-amended soil is still lacking. The main reasons attributed to the paucity of decomposition of BC in soil are insufficient insight to distinguish total soil CO2 efflux from other high CO2 efflux from dead plant residues, root-derived CO2, dissolved OC, soil OM, initial BC stock, and other soil pyrogenic C (Kuzyakov et al., 2009; Wang et al., 2016).
Overall, as a soil amendment, it enhances the biological and physico-chemical characteristics of the soil, especially over a long time, enriching soil aggregation, water holding capacity (WHC), pH, and microbial activity, which enhances overall soil quality. By enhancing the soil’s organic matter content, BC can support sustainable soil management and agricultural productivity. BC acts as a multifunctional soil amendment that not only enhances the soil nutritional profile but also provides a sustainable solution to mitigate the adverse effects of salinity, drought, and heavy metal stressors on agricultural lands.
6 Soil fertility and plant growth enhancement mediated by BC
The frequent application of chemical fertilizers can eventually affect soil fertility, which in turn additionally pollutes adjacent aquatic ecosystems (Jote, 2023). BC application has been an effective way to efficiently reduce the use of synthetic fertilizers, elevate N use efficiency, and promote sustainable agriculture (Gao and DeLuca, 2016). Furthermore, BC promotes plant growth along with higher biomolecule contents, which ensures healthy plantations with nutritionally enhanced crop yields (Tan, 2023). Previously, studies have shown that the nutrient availability to plants and their retention ability in the soil have been improved through enhancing soil CEC and surface oxidation characteristics, which low native organic matter improves soil C stability upon BC amendment (Karimi et al., 2020; Singh et al., 2022). Soil augmented with BC endured higher concentrations of P, N, K, Ca, Mg, and S than untreated soils (Jin et al., 2024; ). The addition of maize residue BC at a rate of 1-2% (w/w) enhanced total N, P, K, copper (Cu), iron (Fe), manganese (Mn) and zinc (Zn) (). Similarly, the application of BC increased the total N, K and P in loamy and clay loamy soils (Nabavinia et al., 2015; Xiao et al., 2016). However, Yao et al. (2017) reported a conflicting result that the addition of maize stalk-derived BC (50 and 200 Mg ha-1) diminished total P and increased total N in soil. The combination and adequate concentration of soil mineral nutrients play a major role in the growth and development of plant species, and nutrient deficiency diminishes plant growth and yield (; Khan et al., 2024). All the reports revealed that the application of BC in soil increased the availability of both macro and micro nutrients.
Apart from improving soil quality, BC enhances seed germination and root development in various plants. For example, seed germination in sweet basil significantly increased by 28% in the 2% BC treatment and 30% in the 3% BC treatment compared with the non-BC control, which depicts a pivotal role of BC in seed germination (Jabborova et al., 2021a). However, improvement in seed germination depends on various factors, such as the type of BC feedstock, rate of BC application, plant species, soil, and other environmental conditions. BC incorporated in soil significantly improves root length, root size, surface area, root diameter, and root volume in apple, strawberry, and sweet basil compared with control plants (Wang et al., 2019; ; Jabborova et al., 2021a). Moreover, increasing (0, 5, 20, and 80 g kg-1) BC dosage application resulted in an increased root respiration of 745, 863, 960, and 1239 nmol O2 min-1 g-1 FW in apple seedlings, respectively (Wang et al., 2019).
BC application enhances plant growth regulators, seed germination, photosynthetic pigments, root growth and soil microbes, which are vital determinants of healthy plant development and productivity and synergistically improve the morphological, physiological, and biochemical properties of plants, soil enzymatic activities and soil fertility. Henceforth, BC may serve as a significant nutritional reservoir for crop development and an efficient amendment to improve soil characteristics.
7 Mechanisms of BC action in alleviating abiotic stresses in soil
Abiotic stresses significantly affect soil health and agricultural productivity. BC has emerged as a promising eco-friendly amendment for enhancing soil nutritional profiles under various abiotic stressors such as salinity, drought, and heavy metal contamination. Amendment of BC in saline soils enhances mineral nutrient, physical, chemical, and biological characteristics of the soil. BC boosts the availability of mineral nutrients and metabolism, EC, infiltration rate, BD, microbial biomass C and pH of the soil under saline-affected soils (Singh et al., 2022). BC ameliorates the adverse salinity effects by balancing WHC, porosity, and its high salt adsorption capabilities (). Specifically, in salt-stressed conditions, BC application was found to notably increase rice biomass through improving soil properties, nutrient conditions and reducing salinity indices like EC, soluble Na+, and Cl- concentrations (Huang et al., 2022). Further, BC has shown to mitigate salinity and drought stress by improving soil structure, increasing water retention capacity, and enhancing the availability of water to plants. It alters the ionic balance in soil, reducing the uptake of Na+ ions under saline conditions and thereby promoting plant growth under stress (Zhang et al., 2013).
BC aids in preserving soil nutrients by diminishing nutrient leaching, in sandy and significantly weathered soils. The higher BC surface area and porosity serve as adhesion sites for nutrients. BC augments soil CEC, substitutes detrimental Na+ ions with beneficial K and Mg ions plays a crucial role in diminishing soil salinity (). Hence, it improves retaining of vital nutrients like K, Ca, and Mg availability to plants. The alkaline pH of BC plays a significant role in neutralizing acidic soils, thereby unravelling nutrients that are naturally inaccessible in acidic environments. The application of BC enhances the soil WHC, pH, CEC and decreases BD contributing to the reduction of heavy metals’ bioavailability and the alleviation of stress caused by salinity and drought (Kumari et al., 2020; Li et al., 2021a).
By increasing the soil pH, BC renders the soil environment more beneficial for plant and microbes. The adjustment of pH facilitates the solubility of nutrients that are less available under acidic conditions, such as P, and helps in reducing the toxicity of aluminium (Al), which causes problem in low pH soils (Huang et al., 2023). BC potentially mitigates heavy metals in saline soil through increasing soil organic C, microbial and biochemical activities (). The synergy between BC and soil organic matter is pivotal for stable soil aggregates formation that facilitates root penetration and improves water infiltration. Furthermore, BC porosity enriches soil porosity, BD, soil structure and water retention that alleviates plants’ resilience to drought conditions (Mukherjee and Lal, 2013).
Immobilization of heavy metals occurs through adsorption on BC surface, complexation with functional groups, and precipitation as metal-BC complexes, thereby mitigating the toxic effects of lead (Pb), cadmium (Cd), and chromium (Cr) in contaminated soils (). BC application is crucial for restoring the productivity of soils affected by industrial pollution and mining activities. BC significantly diminishes metal uptake by plants, as evidenced by lower concentrations of metals in plant tissues.
The ability of BC to enrich nutrient retention in soil is largely attributed to its unique surface functional groups and porosity. The carboxyl, hydroxyl, and phenolic functional groups on BC’s surface are pivotal for enhancing the soil’s ability to retain nutrients, particularly under nutrient-stressed conditions (Hagemann et al., 2017; Pandit et al., 2018). BC functional groups with its porous structure significantly regulates soil P, and N retention by influencing microbial dynamics, which is vital for plant growth (Ibrahim et al., 2020; Zhang et al., 2021). BC can protect organic matter from decomposition, leading to increased soil C sequestration. This stabilization of OM contributes to the long-term improvement of soil fertility, structure, and nutrient cycling (Figure 3).
Figure 3
8 Role of BC in mitigating various abiotic stresses for plant growth and development
Abiotic stresses have been the main constraints for crop production in recent years. For several decades, plant researchers have used various techniques to mitigate abiotic stresses for plant growth and development. In recent years, many researchers have suggested that the application of BC in soil helps to alleviate different abiotic stresses and supports the enhancement of plant growth and yield. Therefore, BC is called “black gold” for agriculture. In this section, we discuss the role of BC in crop improvement under drought, salinity, and heavy metal conditions. Figure 4 is a visual demonstration of the positive impact of BC application on plants grown under normal and different abiotic stresses.
Figure 4
8.1 Salinity stress
Higher concentrations of salt in soil induce osmotic stress due to ionic imbalance, which causes severe effects on morphology, biomass, yield, and biochemical processes in plants (). Salinity stress affects over 1000 million hectares of agricultural land worldwide, making it a serious threat to agriculture (). Therefore, eco-friendly technology is urgently needed to alleviate salinity stress in soil, which helps to improve crop growth and yield. BC enhanced plant biomass, root length, root volume, yield, leaf functional traits and K+ concentration in soybean, tomato (Solanum lycopersicum) and potato (Solanum tuberosum) under salinity stress (; Farhangi-Abriz and Torabian, 2018a; She et al., 2018). Studies by , demonstrated that BC treatment improved growth, biomass and yield traits of rice as well as soil properties (including nutrients availability) under saline conditions. Kanwal et al. (2018) found that applying BC increased the length of root and shoot, leaf functional traits and osmotic potential but decreased the proline content, superoxide dismutase activity and soluble sugar upon salinity stress. BC alleviated salt stress by maintaining higher leaf relative water content (RWC) and a lower Na+/K+ ratio and further enhanced the plant growth, biomass, photosynthesis, transpiration rate and grain quality of rice, sorghum (Sorghum bicolor), maize and wheat (; Huang et al., 2019; Ibrahim et al., 2020, 2021). In another study, BC increased the plant stomatal conductance, plant yield, and chlorophyll fluorescence parameters and reduced abscisic acid in salinity stress-exposed cabbage (). In addition, BC has high salt uptake ability, thus reducing Na+ uptake in plants and mitigating the adverse impact of soil salinity (Huang et al., 2019; Yang et al., 2020).
The role of BC in response to salinity stress in plant growth and metabolism has been extensively studied (Table 3). Overall, it can be concluded that BC can be a useful strategy to alleviate the harmful effects of salinity on plant development. However, BC rates must be carefully used in saline soil to reduce saline toxicity and enhance plant growth processes. The role of BC in physiological and biochemical responses under salt stress has not been studied in many horticultural and economically important plants. Hence, initiating further experiments using BC in other horticultural and economically important plants will help to improve plant quality upon salinity stress, which may help to reduce malnutrition worldwide. Moreover, numerous salinity stress-responsive genes are involved in improving plant growth under salt stress (Golldack et al., 2011; Kumar et al., 2017). The expression pattern and role of salinity stress-related genes have not yet been identified in plants grown under salinity stress with the application of BC. Henceforth, identifying the expression pattern of salt stress-responsive genes in various tissues of plants grown under salinity stress by the application of BC helps to determine which genes are highly induced by BC under salinity stress conditions.
Table 3
| Plant name | Botanical name | Cultivars used | Concentration of NaCl | BC sources | Level of BC | Positive and negative effects of BC | References |
|---|---|---|---|---|---|---|---|
| Potato | Solanum tuberosum | Folva | 25 and 50 mM | Commercial charcoal | 5% | Increased root length, root volume, tuber yield, photosynthetic rate, intrinsic water use efficiency and K+ concentration Decreased leaf water potential, ABA content in xylem sap and leaf, Na+ concentration, leaf Chl content index, total leaf N and C content | |
| Soybean | Glycine max | M7 | 5 and 10 dS m−1 | Sycamore maple plant residues | 50 and 100 g kg−1 | Increased the nodule number and weight, DW of shoot and root, total plant biomass, total plant N, GDH, GS, GOGAT, and NO3- | Farhangi-Abriz and Torabian, 2017 |
| Common bean | Phaseolus vulgaris | Derakhshan | 6 and 12 dS m−1 | Sycamore maple plant residues | 10 and 20% | Increased DW of shoot and root, IAA content of roots Decreased ABA, ACC, JA contents and Na+ content of roots and leaves | Farhangi-Abriz and Torabian, 2018c |
| Derakhshan | 6 and 12 dS m−1 | Sycamore maple plant residues | 5 and 10% | Increased length of root, shoot and leaf area, DW of shoot and root, RWC, Chl fluorescence, Chl-a, Chl-b, total Chl and Chl a/b ratio and various ion concentrations (K+, Ca2+, and Mg2+) in root and shoot tissues Decreased Na+ concentration in shoot and root tissues | Farhangi-Abriz and Torabian, 2018b | ||
| Tomato | Lycopersicon esculentum | Yazhoufenwang | 1 and 3 dS m−1 | Wheat straw | 2, 4 and 8% | Increased photosynthesis and transpiration rate, yield, and number of fruits | She et al., 2018 |
| Wheat | Triticum aestivum | NARC 2009 and NARC 2011 | 150 mM | Wheat leaves | 1 and 2% | Increased root and shoot length, leaf water potential and osmotic potential Decreased proline content, SOD activity and soluble sugar | Kanwal et al., 2018 |
| Sumai-10 | 0.3 and 10 dS m−1 | Wheat straw | 10, 20 and 30 t ha−1 | Increased electrical conductivity, total above-ground biomass, grain yield, harvest index, spike and kernel number, 1000-grain weight, leaf RWC, photosynthesis rate and available P, N and K content in the soil Decreased Na+ concentration | Huang et al., 2019 | ||
| Mung bean | Vigna radiata | MN92 | 5 and 10 dS m-1 | Sycamore maple plant residues | 50 and 100 g kg-1 | Increased root length, root diameter, root DW, root density, specific root length, total root area, shoot DW, shoot/root ratio, root RWC, IAA in root Decreased ABA and ACC content in root | Nikpour et al., 2019 |
| Sorghum | Sorghum bicolor | Kambal | 0.26, 5.8, and 12.6 dS m-1 | Wheat straw | 2.5, 5, and 10% | Increased plant height, leaf area, FW, dry matter yield, photosynthetic rate, stomatal conductance, transpiration rate Decrease activity of CAT, POD, SOD | Ibrahim et al., 2020 |
| Kambal | 0.8, 4.1 and 7.7 dS m−1 | Wheat straw | 2.5, 5, and 10% | Increased shoot and root length, FW and DW of shoot and root and RWC | Ibrahim et al., 2021 | ||
| Eggplant | Solanum melongena | Jaylo | 2 and 4 dS m−1 | Oak and Pine tree woods | 5% | Increased stomatal conductance, photosynthesis rate, density of root length and surface area, plant height, stem diameter, leaf area and yield Decreased leaf temperature and electrolyte leakage in the leaf | Parkash and Singh, 2020 |
| Bonica F1 | 300 mM | Maize straw | 6% | Increased plant height, aerial biomass, fruit number per plant, flowering time and mean FW | Hannachi et al., 2023 | ||
| Quinoa | Chenopodium quinoa | Titicaca | 400 mM | Corn straw | 5% | Increased plant height, shoot biomass, grain yield, leaf photosynthesis, stomatal conductance, intrinsic water use efficiency and leaf K+ Decreased total leaf water potential and ABA content in leaf, leaf Chl content index, leaf N and C content and leaf Na+ content | Yang et al., 2020 |
| Rice | Oryza sativa | G9 | 352.11 mM | Wheat straw | 15, 30 and 45 g per kilogram | Increased biomass, grain yield and quality Decreased Na+ ion accumulation of various tissues | Jin et al., 2018 |
| Changbai-9 | 23.91 dS m− | Rice husk | 30g/kg | Improved rice grain quality traits including amylose content, protein content, taste value, rough rice grain, brown rice rate, white rice rate, whiteness and transmission rate and production | |||
| Jinyuan 85 and Nipponbare | 1 and 3 g kg−1 | Rice straw | – | Decreased electrical conductivity, exchangeable Na+ and exchangeable Cl- | Zhang et al., 2019 | ||
| Changbai-9 | 368.11 mM | Peanut shell | 33.75, 67.5 and 102.5 t ha−1 | Increased leaf water status, plant height, chlorophyll content index and K+ concentration Decreased Na+ concentration, Na+/K+ ratio and leaf-relative electrical leakage | Ran et al., 2020 | ||
| Changbai-9 | 23.91 dS m− | Rice husk | – | Increased plant height, tiller number, dry weight of leaf, panicle, stem and sheath, total dry biomass, K+ concentration and K+/Na+ ratio Improved the concentrations of soil pH, Ca2+, Mg2+, CO32- and Cl- Decreased Na+ concentration in different rice organs and considerably | |||
| Tianlongyou 619 | 4.5 dS m−1 | Maize, wheat and peanut shell residue | 0.5 kg m−2 | Increased plant height, DW, root length, and grain yield Reduced amylose, protein, and taste quality | Zhang et al., 2024 | ||
| Maize | Zea mays | Xianyu335 | 2.0 and 5.0 dS m−1 | Wheat residue | 5 and 10% | Increased plant height, stem diameter, number of leaves per plant, photosynthetic rate, transpiration rate, yield and nutrients N, P, and K uptake | |
| Naudi hybrid | 1.25 and 2.5 g L− 1 | Eucalyptus residues | 50 and 100 g kg− 1 | Increased shoot and root length, DW of shoot and root, Chl a and Chl b, GSTs and CAT activities | Helaoui et al., 2023 | ||
| Cabbage | Brassica olerecae | Yalova1 | 150 mM | Commercial charcoal | 2.5 and 5% | Increased stem diameter, leaf area, FW and DW of root and shoot, leaf RWC, Chl a, Chl b, total Chl and plant nutrient uptake Reduced MDA, H2O2, proline, sucrose Na and Cl content | |
| Shanghai Green | 25, 50, and 100 mM | Corn stover | 2 and 4% | Increased the plant stomatal conductance, plant yield, Chl fluorescence parameters and reduced ABA |
Effects of BC on plant growth and yield under salinity stress in various plants.
RWC, relative water content; DW, dry weight; FW, fresh weight; Chl, chlorophyll; ABA, abscisic acid; ACC,1-aminocyclopropane-1-carboxylic acid content; JA, jasmonic acid; IAA,indole-3-acetic acid; GDH, glutamate dehydrogenase; GS, glutamine synthetase; GSTs, glutathione-S-transferase; GOGAT, glutamine oxoglutarate aminotransferase; SOD, superoxide dismutase; CAT, catalase; POD, peroxidase; MDA, malondialdehyde.
8.2 Drought stress
One of the most important environmental factors affecting the entire plant life cycle was drought. Over 45% of the world’s cultivated land is permanently drought-prone, and 38% of the world’s population lives there (). Therefore, improving water use efficiency in plants exposed to drought stress has long been an important factor in enhancing plant growth and development (Ruggiero et al., 2017). Soil application of BC is considered as an effective practice to facilitate plant growth and yield under drought stress. Many studies have shown that the application of BC in soil increases the growth and yield of drought-stressed plants (Table 4). In tomato, BC increased the soil moisture content, photosynthetic rate, yield, quality of fruit and other biochemical traits under drought stress (; Obadi et al., 2023; Zhang et al., 2023).
Table 4
| Name of the plant | Botanical name | Cultivars used | Drought level | BC sources | Level of BC | Positive and negative effects | References |
|---|---|---|---|---|---|---|---|
| Tomato | Lycopersicon esculentum | No.2 Hongfen | 28% WHC | Mixture of rice husk and shell of cotton seed | 5% | Increased the soil moisture contents, photosynthetic rate, physiology, yield, quality of fruit, RWC, membrane stability index, water use efficiency, stomatal pore aperture and stomatal density Decreased leaf N content and Chl content index and ABA content in leaf | |
| Tone Guitar | 40, 60 and 80% WHC | Date palm fronds waste | 5% | Increased plant height, leaf area index, stem diameter, and FW and DW of above-ground tissues, Chl-a, Chl-b, total Chl, Car contents, water use efficiency and fruit yield | Obadi et al., 2023 | ||
| Ailsa Craig | 70% FC | Wood and poultry manure BC | 5% | Increased plant height, dry mass accumulation, dry root mass, dry leaf mass, ratio of root and shoot, specific leaf area, field WHC and soil water supply Decreased ABA content in xylem sap | Zhang et al., 2023 | ||
| Lady’s Finger | Abelmoschus esculentus | – | 60% FC | Lantana camara plant residues | 1 and 3% | Increased photosynthesis, leaf area, stomatal conductance, dry matter, transpiration rate water use efficiency | |
| Milk thistle | Silybum marianum | – | 40% WHC | Sycamore maple hardwood | 1 and 2% | Increased net photosynthesis rate, water use efficiency, membrane stability index, Chl-a, Chl-b, total Chl, leaf weight, stem weight, leaf area, plant weight and plant height Decreased internal CO2 and stomatal conductance | |
| Soybean | Glycine max | NARC II | – | Corn cobs | 10 and 20 t ha-1 | Increased seedling vigor, germination percentage, rate of germination, membrane stability index of leaf, RWC, shoot length, Chl-a and Chl-b, Car and total Chl Decreased sugar and proline content | Hafeez et al., 2017 |
| Zhonghuang 35 | 40–45% WHC | Wheat straw | 5, and 10 g kg− 1 | Increased water use efficiency, grain yield, root length, root and shoot biomass, photosynthetic rate, stomatal conductance and transpiration rate | Zhang et al., 2020b | ||
| Yeşilsoy | 50, 75 and 100 100% FC | Hazelnut shells | 3 and 6% | Increased plant height, FW and DW of shoot and root, stem diameter, leaf area, Chl-a, Chl-b, total Chl, IAA and GA content Reduced MDA, H2O2, proline, ABA, and sucrose content, and antioxidant activities | Gullap et al., 2024 | ||
| Maize | Zea mays | Amadeo and DKC-3399 | 25–30% WHC | Wood-chip sievings | 1.5 and 3% | Increased above-ground biomass, water use efficiency and soil NO3- content | Haider et al., 2015 |
| ICI-8914 | 40% WHC | – | 4 t ha−1 | Increased DW of shoot and root, length of shoot and root, net photosynthetic rate, transpiration rate, stomatal conductance, Chl-a, Chl-b and Chl a+b | Sattar et al., 2020 | ||
| Wheat | Triticum aestivum | Misr 1 | 50%, 75%, and 100% FC | Corn stalk and rice husk | 1% | Increased Chl-a and Ch- b, Car, RWC, grains per spike, 1000-grain weight, grain yield and harvest index | Hafez et al., 2021 |
| Glaxay 2013 | 30% WHC | Wheat straw | 27.88 and 37.18 g kg-1 | Increased plant height, number of fertile tillers, spike length, number of spikelets per spike, number of grains per spike and 1000-grain weight | Haider et al., 2020 | ||
| Galaxy-2013 | – | Commercial charcoal | 28 g kg−1 and 38 g kg−1 | Plant height, spike length, number of spikelet’s per spike, number of grains per spike, 1000-grain weight, grain yield per plant, N, P and K contents in soil and microbial biomass | Zaheer et al., 2021 | ||
| Galaxy 2013 | 30% WHC | Wheat straw | 3 and 5% | Increased plant height, fertile tiller count, spike length, grains per spike, 1000-grain weight, yield, water use efficiency, stomatal conductance, Chl-a, Chl-b, transpiration rate, photosynthetic rate, electrolyte leakage, H2O2, SOD, CAT and POD | Zulfiqar et al., 2022 | ||
| Cabbage | Brassica olerecae | Yalova1 | 50% WHC | Commercial charcoal | 5 and 10% | Increased FW and DW of shoot and root, Chl-a, Chl-b, total Chl, leaf RWC, CAT, POD and SOD activities and nutrient uptake Decreased H2O2, MDA and proline contents | Yildirim et al., 2021 |
| Eggplant | Solanum melongena | Bonica F1 | >30% WHC | Maize straw | 6% | Increased plant height, aerial biomass, number of fruits per plant, flowering time and mean FW | Hannachi et al., 2023 |
| Melon | Cucumis melo | – | 60, 85, and 100% WHC | Palm leaves | 0.24 and 0.36 kg m-2 | Increased water use efficiency, FW and DW of root and shoot, root length, average fruit weight, fruit diameter, fruit flesh thickness, leaf N, Mn, K, Fe, Zn and Cu contents |
Effects of BC on plant growth and yield under drought stress in various plants.
RWC, relative water content; DW, dry weight; FW, fresh weight; Chl, chlorophyll; Car, carotenoid; ABA, abscisic acid; IAA,indole-3-acetic acid; GA, gibberellic acid; SOD, superoxide dismutase; CAT, catalase; POD, peroxidase; MDA, malondialdehyde; WHC, water holding capacity; FC, field capacity.
BC application enhanced the soil moisture holding capacity, net photosynthesis rate, water use efficiency and physiological, biomass and biochemical traits in milk thistle plants exposed to drought stress (). BC ameliorates drought-stressed soybean growth from the seedling stage to yield, including seed germination and biochemical and physiological traits (Hafeez et al., 2017; Zhang et al., 2020b; Gullap et al., 2024). The combined application of BC and silicon improved biomass- and yield-related traits in maize upon drought stress (Sattar et al., 2020). BC significantly enhanced physiological, biochemical and yield traits related to drought stress tolerance in maize (Hafez et al., 2020; Haider et al., 2020; Zaheer et al., 2021; Zulfiqar et al., 2022). It has been revealed that BC treatment strengthens the defense mechanisms of drought stressed plants. As with salt-stress responsive genes, many drought-tolerant and drought-susceptible genes have been reported in plants (Kaur and Asthir, 2017; Mahmood et al., 2019). The expression pattern and role of drought-tolerant and drought-susceptible genes have not been initiated under drought stress in plants with BC amendment. Hence, in-depth molecular experiments are urgently needed to underpin the expression pattern and role of drought-tolerant and susceptible genes in plants grown under BC.
8.3 Heavy metal stress
Contamination of agricultural soil by pollutants such as heavy metals has become a growing environmental problem worldwide that affects nutrient uptake, plant growth, and metabolism. Various measures have been used to remediate heavy metal contamination from soils, including the use of metal hyper accumulator plants, organic and inorganic amendments, and agricultural practices (Maharajan et al., 2022). Among these, organic amendments are effective techniques and eco-friendly methods to reduce plant uptake of high concentrations of heavy metals from heavy metal-contaminated soils. BC can absorb heavy metals from contaminated soil and reduce their toxic effects on plants. This has been demonstrated in many plant species (Table 5). The application of cotton stalk-derived BC increased growth, biomass, transpiration rate, sub-stomatal CO2 concentrations, photosynthetic rate, chlorophyll and carotenoid contents while reducing Cd concentrations and malondialdehyde content in shoot and root tissue under Cd toxicity (Younis et al., 2016). In a study by Woldetsadik et al. (2016), the application of poultry litter, cow manure, and coffee husk BC immobilized Cd in the soil and reduced the Cd concentration in plant tissues, while BC increased the growth and uptake of P in lettuce plants. In another study, BC deduced concentrations of Cd, Cu, Pb and increased the concentrations of P, Fe and Zn in shoot and root tissues of maize (). Similarly, Miscanthus residues reduced nickel (Ni) contents in root, shoot and grains and increased the dry weight of shoot and root, photosynthetic rate, stomatal conductance, transpiration rate, yield, and several biochemical traits in maize upon Ni stress (Shahbaz et al., 2018).
Table 5
| Name of the plant | Botanical name | Heavy metal level | BC sources | Level of BC | Positive and negative effects | References |
|---|---|---|---|---|---|---|
| Spinach | Spinacia oleracea | Cd (25, 50 and 100 mg kg−1) | Cotton stalks | 3 and 5% | Increased growth, biomass, transpiration rate, substomatal CO2 concentrations, photosynthetic rate, Chl-a, Chl-b, total Chl, protein and Car contents Decreased Cd concentrations and MDA content in shoot and root tissue | Younis et al., 2016 |
| Mn (3.779 ppm), Ni (0.331 ppm), Zn (4.88 ppm), Cr (0.138 ppm) and Mg(111.7 ppm) | Cow manure and fresh sheep/goat manure | 3, 5 and 10% | Increased the leaf area index, above-ground biomass, water use efficiency, root biomass Reduced Ni content in leaves | Tahir et al., 2018 | ||
| Pb (250 mg kg−1) | Waste material of vegetables and fruits | 0.5% | Increased FW and DW weight of root and K contents Reduced Pb content in root | Zafar-ul-Hye et al., 2020 | ||
| Lettuce | Lactuca sativa | Cd (50 mg kg−1) | Poultry litter, cow manure and coffee husk | 7% | Increased plant growth, yield, and P uptake Reduced Cd concentration | Woldetsadik et al., 2016 |
| Wheat | Triticum aestivum | Cd (2.86 mg kg−1), Zn (47.29 mg kg−1), Mn (68.31 mg kg−1) and Ni (5.33 mg kg−1) | Rice straw | 1.5, 3.0 and 5.0% | Increased plant height, spike length, root, spike, grain and shoot biomass, grain yield, photosynthetic rate, Chl-a, Chl-b, transpiration rate, stomatal conductance, water use efficiency, Zn and Mn concentrations in shoots, roots, and grains and Si content, activities of SOD, CAT in shoot and root Decreased the Cd and Ni contents in shoot, root and grains and MDA content in shoot and root | |
| Tomato | Solanum lycopersicum | Cd (0.13 and 2 μg/ml) | Cotton stalk | 1% | Increased soil pH, soil electronic conductivity, soil organic matter, DW of shoot and root, length of root and stem, Chl-a, Chl-b, total Chl, anthocyanin, Car and lycopene contents Reduced total Cd in soil, shoot Cd concentration | |
| Maize | Zea mays | Cu (3474 mg kg−1) Fe (25 962 mg kg−1) Mn (1413 mg kg−1) Pb (1360 mg kg−1) Zn (11 239 mg kg−1) Cd (27.8 mg kg−1) | Date palm tree waste | 1, 2 and 3% | Increased P, Fe and Zn concentration in shoot and root Reduced Cd, Cu, Pb concentration in shoot and root tissue | |
| Ni (77 mg kg−1) | Miscanthus plant residues | 2% | Increased DW of shoot and root, grain yield, photosynthetic rate, stomatal conductance, transpiration rate, CAT, APX and DHAR activities, ABA in leaves, protein, fiber, fat, starch Reduced MDA and H2O2 activities in leaf and polyphenol, Ni contents in root, shoot and grains | Shahbaz et al., 2018 | ||
| Chinese cabbage | Brassica chinensis | Cd (41 mg kg−1) | Rice straw, rice hull and maize stover | 1.5 and 3% | Increased FW and DW of shoot and root, length of shoot, root and leaves Reduced Cd content in shoot and root tissue | |
| Cd (20 mg kg−1) | Wheat straw | 5% | Increased plant biomass Reduced Cd contents in fruits | Sun et al., 2020 | ||
| Chinese flowering cabbage | Brassica parachinensis | Cd (1.19 mg kg−1) | Pennisetum hydridum straws | 2% | Increased vegetable growth, plant height, root length, root FW, above-ground FW and reduced Cd content in the roots and above ground tissues | Li et al., 2021b |
| Sunflower | Helianthus annuus | Ni (77 mg kg−1) | Miscanthus residues | 2% | Increased DW of shoot and root, grain yield, photosynthetic rate, stomatal conductance, transpiration rate, CAT, APX and DHAR activities, ascorbic acid in leaves, protein, fiber, fat, starch Reduced MDA and hydrogen peroxide activities in leaf and polyphenol, Ni contents in root, shoot and grains | Shahbaz et al., 2018 |
| Pea | Pisum sativum | Pb (1000 mg kg−1) | – | 2% | Increased DW of shoot and root, grain yield, plant height, RWC, Chl-a, Chl-b, protein, fat, fiber, carbohydrate, Fe, Zn and Mn contents, APX, SOD, CAT and DHAR activities Reduced Pb content in root and shoot and polyphenols, MDA, H2O2 and O2 | Haider et al., 2019 |
| Peanuts | Arachis hypogaea | Cd (1 mg kg−1) | Peanut vine and rice straw | 5% | Increased soil pH, Chl content, soluble sugars, proline, soluble protein and crude fat Reduced Cd content in the root, above-ground tissues, shell and seed | |
| Rapeseed | Brassica napus | Cd (0.28 mg kg−1), Cr (11.30 mg kg−1), Cu (3.60 mg kg−1), Zn (17.94 mg kg−1), Ni (1.38 mg kg−1), Pb (5.84 mg kg−1), Co (0.10 mg kg−1) and Fe (136.38 mg kg−1) | Acacia nilotica woodchip | 1 and 2% | Increased FW of shoot and root, Chl-a, Chl-b, total Chl, total pigments, Car, lycopene concentration, APX, POD and CAT activities. Reduced Cd, Pb, Ni and Cu in soil and shoot and roots | Kamran et al., 2020 |
| Barley | Hordeum vulgare | Cd (1.25-1.91 mg kg−1), Cu (200-451 mg kg−1), Pb (118-211 mg kg−1) and Zn (67.2-134 mg kg−1) | Miscanthus residues | 2% | Increased shoot and root biomass and reduced Cu, Pb, Cd and Zn contents in shoot and root tissues | Medynska et al., 2020 |
| Green pepper | Capsicum annuum | Cd (20 mg kg−1) | Wheat straw | 5% | Increased plant biomass and reduced Cd contents in fruits | Sun et al., 2020 |
| Eggplant | Solanum melongena | Cd (20 mg kg−1) | Wheat straw | 5% | Increased plant biomass and reduced Cd contents in fruits | Sun et al., 2020 |
Effects of BC on plant growth and yield under heavy metal stress in various plants.
DW, dry weight; FW, fresh weight; Chl, chlorophyll; Car, carotenoid; ABA, abscisic acid; APX, ascorbate peroxidase; DHAR, dehydrogenase reductase; SOD, superoxide dismutase; CAT, catalase; POD, peroxidase; MDA, malondialdehyde.
BC derived from wheat straw increased plant biomass and reduced Cd contents in fruits of green pepper and eggplant (Sun et al., 2020). Overall, BC could be effective in immobilizing heavy metals in the soil and reducing heavy metal uptake and accumulation in plant tissues. In general, HM uptake by roots is facilitated by various metal transporters (Maharajan et al., 2022). However, the role of heavy metal transporters has not yet been reported in BC-treated plant tissues. Hence, environmental researchers should collaborate with plant molecular biologists to initiate in-depth molecular experiments in this field, which may help to understand the accurate role of BC in plant growth and yield. Apart from this, BC derived from heavy metal accumulator plant residues has not yet been used for any experiments. Hence, researchers can try to derive BC from heavy metal accumulator plant tissues and apply them to identify the effect of BC on plant growth and yield.
9 Conclusion and future perspectives
The utilization of BC, derived from agricultural and forestry residues, aligns with global sustainability goals by converting waste materials into valuable resources that enhance agricultural output. Synthesis techniques, BC processing, soil amendments, and applications to alleviate abiotic stressors in plants have received a lack of research attention. Hence, this review compiles the conversion of residual biomass into valuable BC amendments for soil and crop improvement upon abiotic stressors. Due to the post pandemic financial crisis, low-cost soil amendments are mandatory to increase crop production to overcome worldwide food scarcity. BC application is a promising strategy to promote soil–plant enrichment for the production of highly nutritious crops and yields, ameliorate plant abiotic stresses, controlled usage of hazardous synthetic fertilizer-based soil amendments to enhance sustainable agriculture. BC has a positive impact on soil structure, quality, and physico-chemical properties such as BD, pH, CEC, porosity, nutrient balance, WHC, and aeration. The optimal ratio of BC formulations has been potentially enriching yields under plant- and soil-specific constraints, limited water, nutrients and adverse conditions. Also, offering a promising avenue for enhancing global food security and environmental health. The recommended dosage of BC for quality improvement under specific soil and plant species is not yet well defined. Moreover, research must be focused on BC at low doses, and high efficacy is crucial to maximize farmer-friendly, cost-effective BC applications for several cropping systems.
The synergistic effects of BC along with compost, fertilizers and beneficial soil microbes that stimulate crop growth and soil fertility remain unclear. Although, long-term BC risk management and life cycle assessments are not yet completely clarified. The discrepancy between field and laboratory experiments regarding physico-chemical properties, soil quality, abiotic stress, environmental impacts, and plant growth efficiency should be scrutinized. BC production parameter optimization, functionalization, elucidation of BC augmenting mechanisms, integration of multi-omics technologies, data-driven and machine learning methods would contribute to BC applications for soil fertility and cost-effective high-yielding production of valuable crops in sustainable agricultural management. While initial production and application costs can be high, the long-term savings, enhanced crop resilience, and potential carbon credits make BC a viable option. However, further technological advancements and policy support are essential to encourage broader adoption. As per our knowledge, physiological and biochemical modifications by BC under abiotic stress have been identified, while molecular identification and characterization in this field remain underexplored. These areas of research should be prioritized by plant and environmental scientists, as they could provide deeper insights into plant development, food security, and sustainable agricultural practices. In summary, increasing soil health along with sustainable crop productivity and profitability under challenging environmental conditions can be significantly influenced by BC soil amendment technologies. Moreover, additional investigation is required to implement the machine learning approach on BC-based soil amendment, the alleviation of abiotic stress for sustainable crop production, soil fertility management, and hence light up BC industrialization.
Statements
Author contributions
PR: Formal analysis, Investigation, Resources, Software, Writing – original draft. TM: Data curation, Visualization, Writing – original draft. RJ: Writing – review & editing. MP: Writing – review & editing. IL: Data curation, Investigation, Resources, Writing – review & editing. PY: Data curation, Investigation, Resources, Writing – review & editing. SJ: Funding acquisition, Project administration, Supervision, Writing – review & editing.
Funding
The author(s) declare financial support was received for the research, authorship, and/or publication of this article. This work was supported by the “Cooperative Research Program for Agriculture Science and Technology Development (Project No. RS-2020-RD008517)” Rural Development Administration, Republic of Korea. This work was supported by the 2023 RDA Fellowship program of the National Institute of Horticultural and Herbal Science, Rural Development Administration, Republic of Korea.
Acknowledgments
We would like to express sincere gratitude to Dr. Subramani Pandian, Dr. Pandian Muthuramalingam, Dr. Subramanian Muthamil and Dr. Jayabalan Shilpha for helping during the study.
Conflict of interest
The authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.
Publisher’s note
All claims expressed in this article are solely those of the authors and do not necessarily represent those of their affiliated organizations, or those of the publisher, the editors and the reviewers. Any product that may be evaluated in this article, or claim that may be made by its manufacturer, is not guaranteed or endorsed by the publisher.
References
1
AbbasT.RizwanM.AliS.Zia-ur-RehmanM.QayyumM. F.AbbasF.et al. (2017). Effect of biochar on cadmium bioavailability and uptake in wheat (Triticum aestivum L.) grown in a soil with aged contamination. Ecotoxicol. Environ. Contam.140, 37–47. doi: 10.1016/j.ecoenv.2017.02.028
2
AbidM.DanishS.Zafar-ul-HyeM.ShaabanM.IqbalM. M.RehimA.et al. (2017). Biochar increased photosynthetic and accessory pigments in tomato (Solanum lycopersicum L.) plants by reducing cadmium concentration under various irrigation waters. Environ. Sci. pollut. Res.24, 22111–22118. doi: 10.1007/s11356-017-9866-8
3
AdekiyaA. O.AgbedeT. M.OlayanjuA.EjueW. S.AdekanyeT. A.AdenusiT. T.et al. (2020). Effect of biochar on soil properties, soil loss, and cocoyam yield on a tropical sandy loam Alfisol. Sci. World. J., 9391630. doi: 10.1155/2020/9391630
4
AdelawonB. O.LatinwoG. K.EboibiB. E.AgbedeO. O.AgarryS. E. (2022). Comparison of the slow, fast, and flash pyrolysis of recycled maize-cob biomass waste, box-benhken process optimization and characterization studies for the thermal fast pyrolysis production of bio-energy. Chem. Commun.209, 1246–1247. doi: 10.1080/00986445.2021.1957851
5
AdhikariU.NejadhashemiA. P.WoznickiS. A. (2015). Climate change and eastern Africa: a review of impact on major crops. Food. Energy. Secur.4, 110–132. doi: 10.1002/fes3.61
6
AfsharK. R.HashemiM.DaCostaM.SpargoJ.SadeghpourA. (2016). Biochar application and drought stress effects on physiological characteristics of Silybum marianum. Commun. Soil. Sci. Plant Anal.47, 743–752. doi: 10.1080/00103624.2016.1146752
7
AgegnehuG.SrivastavaA. K.MichaelI. (2017). The role of biochar and biochar-compost in improving soil quality and crop performance: A review. Appl. Soil. Ecol.119, 156–170. doi: 10.1016/j.apsoil.2017.06.008
8
AhmadM.UsmanA. R.Al-FarajA. S.AhmadM.SallamA.Al-WabelM. I. (2018). Phosphorus-loaded biochar changes soil heavy metals availability and uptake potential of (Zea mays L.) plants. Chemosphere194, 327–339. doi: 10.1016/j.chemosphere.2017.11.156
9
AjorlooM.GhodratM.ScottJ.StrezovV. (2022). Recent advances in thermodynamic analysis of biomass gasification: A review on numerical modelling and simulation. J. Energy. Inst.102, 395–419. doi: 10.1016/j.joei.2022.05.003
10
AkhtarS. S.AndersenM. N.LiuF. (2015). Biochar mitigates salinity stress in potato. J. Agron. Crop Sci.201, 368–378. doi: 10.1111/jac.12132
11
AkhtarS. S.LiG.AndersenM. N.LiuF. (2014). Biochar enhances yield and quality of tomato under reduced irrigation. Agric. Water. Manage.138, 37–44. doi: 10.1016/j.agwat.2014.02.016
12
AlfadilA. A.XiaJ.ShaghalehH.Alhaj HamoudY.IbrahimJ. N.HamadA. A. A.et al. (2021). Wheat straw biochar application improves the morphological, physiological, and yield attributes of maize and the physicochemical properties of soil under deficit irrigation and salinity stress. J. Plant Nutr.44, 2399–2420. doi: 10.1080/01904167.2021.1918156
13
AlkharabshehH. M.SeleimanM. F.BattagliaM. L.ShamiA.JalalR. S.AlhammadB. A.et al. (2021). Biochar and its broad impacts in soil quality and fertility, nutrient leaching and crop productivity: A review. Agronomy11, 5–993. doi: 10.3390/agronomy11050993
14
AmbayeT. G.VaccariM.van HullebuschE. D.AmraneA.RtimiS.J.I.J.O.E.S. (2021). Mechanisms and adsorption capacities of biochar for the removal of organic and inorganic pollutants from industrial wastewater. Inter. J. Environ. Sci. Technol.18, 3273–3294. doi: 10.1007/s13762-020-03060-w
15
AmelootN.GraberE. R.VerheijenF. G.De NeveS. (2013). Interactions between biochar stability and soil organisms: review and research needs. Euro. J. Soil Sci.64, 379–390. doi: 10.1111/ejss.12064
16
AnwariG.FengJ.MoussaA. A. (2019a). Multiple beneficial effects of using biochar (as a great organic material) on tolerance and productivity of rice under abiotic stress. J. Mod. Mat.6, 40–51. doi: 10.21467/jmm.6.1.40-51
17
AnwariG.TianxuY.Alio MoussaA.WentaoZ.MandozaiA.GamalM.et al. (2023). Influence of biochar and aluminum sulfate on rice growth and production in saline soil. J. Crop Imp.37, 776–795. doi: 10.1080/15427528.2022.2151541
18
AnwariG.XiaoxuanH.YimingZ.TianxuY.WenanW.BowenZ.et al. (2019b). Effects of rice-husk biochar and aluminum sulfate application on rice grain quality in saline-sodic soil of paddy-field. Int. J. Biosci.15, 325–333. doi: 10.12692/ijb/15.6.325-333
19
AwogbemiO.KallonD. V. V. (2023). Application of biochar derived from crops residues for biofuel production. Fuel. Commun.15, 100088. doi: 10.1016/j.jfueco.2023.100088
20
AzadiN.RaiesiF. (2021). Salinization depresses soil enzyme activity in metal-polluted soils through increases in metal mobilization and decreases in microbial biomass. Ecotoxicology30, 1071–1083. doi: 10.1007/s10646-021-02433-2
21
BagheriS.HassandokhtM. R.MirsoleimaniA.MousaviA. (2019). Effect of palm leaf biochar on melon plants (Cucumis melo L.) under drought stress conditions. Adv. Hortic. Sci.33, 593–604. doi: 10.13128/ahsc8228
22
BalasubramaniamT.ShenG.EsmaeiliN.ZhangH. (2023). Plants’ response mechanisms to salinity stress. Plants12, 12–2253. doi: 10.3390/plants12122253
23
BashirS.HussainQ.ShaabanM.HuH. (2018). Efficiency and surface characterization of different plant derived biochar for cadmium (Cd) mobility, bioaccessibility and bioavailability to Chinese cabbage in highly contaminated soil. Chemosphere211, 632–639. doi: 10.1016/j.chemosphere.2018.07.168
24
BatoolA.TajS.RashidA.KhalidA.QadeerS.SaleemA. R.et al. (2015). Potential of soil amendments (Biochar and Gypsum) in increasing water use efficiency of Abelmoschus esculentus L. Moench. Front. Plant Sci.6. doi: 10.3389/fpls.2015.00733
25
BekchanovaM.CampionL.BrunsS.KuppensT.LehmannJ.JozefczakM.et al. (2024). Biochar improves the nutrient cycle in sandy-textured soils and increases crop yield: a systematic review. Environ. Evi.13, 3. doi: 10.1186/s13750-024-00326-5
26
BibiS.UllahS.HafeezA.KhanM. N.JavedM. A.AliB.et al. (2022). Exogenous Ca/Mg quotient reduces the inhibitory effects of PEG induced osmotic stress on Avena sativa L. Braz. J. Biol.84, e264642. doi: 10.1590/1519-6984.264642
27
BiloF.PandiniS.SartoreL.DeperoL. E.GargiuloG.BonassiA.et al. (2018). A sustainable bioplastic obtained from rice straw. J. Clean. Prod.200, 357–368. doi: 10.1016/j.jclepro.2018.07.252
28
BolanS.HouD.WangL.HaleL.EgamberdievaD.TammeorgP.et al. (2023). The potential of biochar as a microbial carrier for agricultural and environmental applications. Sci. Total. Environ., 163968. doi: 10.1016/j.scitotenv.2023.163968
29
BoostaniH. R.HardieA. G.Najafi-GhiriM. (2020). Effect of organic residues and their derived biochars on the zinc and copper chemical fractions and some chemical properties of a calcareous soil. Commun. Soil. Sci. Plant Analy.51, 1725–1735. doi: 10.1080/00103624.2020.1798986
30
ButcherK.WickA. F.DeSutterT.ChatterjeeA.HarmonJ. (2016). Soil salinity: A threat to global food security. Agronomy J.108, 2189–2200. doi: 10.2134/agronj2016.06.0368
31
CaoX.MaL.LiangY.GaoB.HarrisW. (2011). Simultaneous immobilization of lead and atrazine in contaminated soils using dairy-manure biochar. Environ. Sci. Technol.45, 4884–4889. doi: 10.1021/es103752u
32
ChausaliN.SaxenaJ.PrasadR. (2021). Nanobiochar and biochar based nanocomposites: Advances and applications. J. Agricul. Food Res.5, 100191. doi: 10.1016/j.jafr.2021.100191
33
ChenX.HeH. Z.ChenG. K.LiH. S. (2020). Effects of biochar and crop straws on the bioavailability of cadmium in contaminated soil. Sci. Rep.10, 9528. doi: 10.1038/s41598-020-65631-8
34
ChenY.SunK.YangY.GaoB.ZhengH. (2023). Effects of biochar on the accumulation of necromass-derived carbon, the physical protection and microbial mineralization of soil organic carbon. Critical Rev. Environ. Sci. Technol.54, 1–29. doi: 10.1080/10643389.2023.2221155
35
ChiN. T. L.AntoS.AhamedT. S.KumarS. S.ShanmugamS.SamuelM. S.et al. (2021). A review on biochar production techniques and biochar based catalyst for biofuel production from algae. Fuel287, 119411. doi: 10.1016/j.fuel.2020.119411
36
ChintalaR.SchumacherT. E.McDonaldL. M.ClayD. E.MaloD. D.PapiernikS. K.et al. (2014). Phosphorus sorption and availability from biochars and soil/biochar mixtures. CLEAN Soil Air Water.42, 626–634. doi: 10.1002/clen.201300089
37
ChiomentoJ. L. T.De NardiF. S.FilippiD.dos Santos TrentinT.DornellesA. G.FornariM.et al. (2021). Morpho-horticultural performance of strawberry cultivated on substrate with Arbuscular mycorrhizal fungi and biochar. Sci. Hortic.282, 110053. doi: 10.1016/j.scienta.2021.110053
38
ChoS. H.LeeS.KimY.SongH.LeeJ.TsangY. F.et al. (2023). Applications of agricultural residue biochars to removal of toxic gases emitted from chemical plants: A review. Sci. Total. Environ.868, 161655. doi: 10.1016/j.scitotenv.2023.161655
39
ChoudharyT. K.KhanK. S.HussainQ.AshfaqM. (2021). Nutrient availability to maize crop (Zea mays L.) in biochar amended alkaline subtropical soil. J. Soil Sci. Plant Nutr.21, 1293–1306. doi: 10.1007/s42729-021-00440-0
40
DafiqurrohmanH.SafitriK. A.SetyawanM. I. B.SurjosatyoA.AzizM. (2022). Gasification of rice wastes toward green and sustainable energy production: A review. J. Clean. Prod.366, 132926. doi: 10.1016/j.jclepro.2022.132926
41
DalalR. C.AllenD. E.ChanK. Y.SinghB. P. (2011). “Soil organic matter, soil health and climate change, soil health and climate change,” in Soil Health and Climate Change. Soil Biol., vol. Vol 29 . Eds. SinghB.CowieA.ChanK. (Springer, Berlin, Heidelberg), 87–106. doi: 10.1007/978-3-642-20256-8_5
42
DasS.NewarR.SaikiaA.BaruahA. (2023). “Biomass-based engineered materials for soil remediation,” in Land Remediation and Management: Bioengineering Strategies (Springer Nature Singapore, Singapore), 253–293. doi: 10.1007/978-981-99-4221-3_12
43
DasR.PandaS. N. (2022). Preparation and applications of biochar based nanocomposite: A review. J. Anal. Appl. Pyrol.167, 105691. doi: 10.1016/j.jaap.2022.105691
44
De Jesus DuarteS.GlaserB.Pellegrino CerriC. E. (2019). Effect of biochar particle size on physical, hydrological and chemical properties of loamy and sandy tropical soils. Agronomy9, 165. doi: 10.3390/agronomy9040165
45
De VasconcelosA. C. F. (2020). Biochar effects on amelioration of adverse salinity effects in soils. Appl. Biochar Environ. Saf.12, 193–204.
46
DingY.LiuY.LiuS.LiZ.TanX.HuangX.et al. (2016). Biochar to improve soil fertility. A review. Agron. Sustain Dev.36, 1–18. doi: 10.1007/s13593-016-0372-z
47
DongM.HeL.JiangM.ZhuY.WangJ.GustaveW.et al. (2023). Biochar for the removal of emerging pollutants from aquatic systems: a review. Int. J. Environ. Res. Public Health20, 1679. doi: 10.3390/ijerph20031679
48
EkinciM.TuranM.YildirimE. (2022). Biochar mitigates salt stress by regulating nutrient uptake and antioxidant activity, alleviating the oxidative stress and abscisic acid content in cabbage seedlings. Turkish J. Agric. Fores.46, 28–37. doi: 10.3906/tar-2104-81
49
El-NaggarA.LeeS. S.AwadY.XiaoY.RyuC.RinklebeJ.et al. (2018). Influence of soil properties and feedstocks on biochar potential for carbon mineralization and improvement of infertile soils. Geoderma332, 100–108. doi: 10.1016/j.geoderma.2018.06.017
50
FahadS.BajwaA. A.NazirU.AnjumS. A.FarooqA.ZohaibA.et al. (2017). Crop production under drought and heat stress: plant responses and management options. Front. Plant Sci.8. doi: 10.3389/fpls.2017.01147
51
FahmyT. Y.FahmyY.MobarakF.El-SakhawyM.Abou-ZeidR. E. (2020). Biomass pyrolysis: past, present, and future. Environ. Dev. Sustain.22, 17–32. doi: 10.1007/s10668-018-0200-5
52
FAO (2022). FAOSTAT: Production: Crops and livestock products (Rome: FAO). Available at: https://www.fao.org/faostat/en/data/QCL (Accessed April 21, 2024).
53
Farhangi-AbrizS.TorabianS. (2017). Antioxidant enzyme and osmotic adjustment changes in bean seedlings as affected by biochar under salt stress. Ecotoxicol. Environ. Saf.137, 64–70. doi: 10.1016/j.ecoenv.2016.11.029
54
Farhangi-AbrizS.TorabianS. (2018a). Biochar improved nodulation and nitrogen metabolism of soybean under salt stress. Symbiosis74, 215–223. doi: 10.1007/s13199-017-0509-0
55
Farhangi-AbrizS.TorabianS. (2018b). Biochar increased plant growth-promoting hormones and helped to alleviates salt stress in common bean seedlings. J. Plant Growth Regul.37, 591–601. doi: 10.1007/s00344-017-9756-9
56
Farhangi-AbrizS.TorabianS. (2018c). Effect of biochar on growth and ion contents of bean plant under saline condition. Environ. Sci. pollut. Res.25, 11556–11564. doi: 10.1007/s11356-018-1446-z
57
FrydaL.VisserR. (2015). Biochar for soil improvement: Evaluation of biochar from gasification and slow pyrolysis. Agric5, 1076–1115. doi: 10.3390/agriculture5041076
58
GabhaneJ. W.BhangeV. P.PatilP. D.BankarS. T.KumarS. (2020). Recent trends in biochar production methods and its application as a soil health conditioner: a review. SN Appl. Sci.2, 1307. doi: 10.1007/s42452-020-3121-5
59
GaoS.DeLucaT. H. (2016). Influence of biochar on soil nutrient transformations, nutrient leaching, and crop yield. Adv. Plants Agric. Res.4, 348–362. doi: 10.15406/apar.2016.04.00150
60
GaoS.Hoffman-KrullK.BidwellA. L.DeLucaT. H. (2016). Locally produced wood biochar increases nutrient retention and availability in agricultural soils of the San Juan Islands, USA. Agric. Ecosyst. Environ.233, 43–54. doi: 10.1016/j.agee.2016.08.028
61
GarlapalliR. K.WirthB.RezaM. T. (2016). Pyrolysis of hydrochar from digestate: Effect of hydrothermal carbonization and pyrolysis temperatures on pyrochar formation. Biores. Technol.220, 168–174. doi: 10.1016/j.biortech.2016.08.071
62
GlaserB.LehmannJ.ZechW. (2002). Ameliorating physical and chemical properties of highly weathered soils in the tropics with charcoal–a review. Biol. Fertil Soils35, 219–230. doi: 10.1007/s00374-002-0466-4
63
GodlewskaP.SchmidtH. P.OkY. S.OleszczukP. (2017). Biochar for composting improvement and contaminants reduction. A review. Biores. Technol.246, 193–202. doi: 10.1016/j.biortech.2017.07.095
64
GollakotaA.KishoreN.GuS. (2018). A review on hydrothermal liquefaction of biomass. Renew. Sustain. Energy. Rev.81, 1378–1392. doi: 10.1016/j.rser.2017.05.178
65
GolldackD.LükingI.YangO. (2011). Plant tolerance to drought and salinity: stress regulating transcription factors and their functional significance in the cellular transcriptional network. Plant Cell. Rep.30, 1383–1391. doi: 10.1007/s00299-011-1068-0
66
Gonzalez-PernasF. M.Grajera-AntolínC.García-CámaraO.González-LucasM.MartínM. T.González-EgidoS.et al. (2022). Effects of biochar on biointensive horticultural crops and its economic viability in the Mediterranean climate. Energies15, 9–3407. doi: 10.3390/en15093407
67
GoyalD.YadavA.PrasadM.SinghT. B.ShrivastavP.AliA.et al. (2020). “Effect of heavy metals on plant growth: an overview,” in Contaminants in Agriculture. Eds. NaeemM.AnsariA.GillS. (Springer, Cham). doi: 10.1007/978-3-030-41552-5_4
68
GranatsteinD.KrugerC.CollinsH.Garcia-PerezM.YoderJ. (2009). Use of biochar from the pyrolysis of waste organic material as a soil amendment. Final Project Report (Wenatchee, WA: Center for Sustaining Agriculture and Natural Resources, Washington State University). Available at: https://hdl.handle.net/2376/5869 (Accessed April 21, 2024).
69
GriffithS. M.BanowetzG. M.GadyD. (2013). Chemical characterization of chars developed from thermochemical treatment of Kentucky bluegrass seed screenings. Chemosphere92, 1275–1279. doi: 10.1016/j.chemosphere.2013.02.002
70
GullapM. K.SeverogluS.KarabacakT.YaziciA.EkinciM.TuranM.et al. (2024). Biochar derived from hazelnut shells mitigates the impact of drought stress on soybean seedlings. New Zealand. J. Crop Hortic. Sci.52, 1–19. doi: 10.1080/01140671.2022.2079680
71
GuoY.RockstrawD. A. (2007). Physicochemical properties of carbons prepared from pecan shell by phosphoric acid activation. Biores. Technol.98, 1513–1521. doi: 10.1016/j.biortech.2006.06.027
72
GuptaB.ShresthaJ. (2023). Editorial: Abiotic stress adaptation and tolerance mechanisms in crop plants. Front. Plant Sci.14. doi: 10.3389/fpls.2023.1278895
73
HafeezY.IqbalS.JabeenK.ShahzadS.JahanS.RasulF. (2017). Effect of biochar application on seed germination and seedling growth of Glycine max (L.) Merr. Under drought stress. Pakistan J. Bot.49, 7–13.
74
HafezY.AttiaK.AlameryS.GhazyA.Al-DossA.IbrahimE.et al. (2020). Beneficial effects of biochar and chitosan on antioxidative capacity, osmolytes accumulation, and anatomical characters of water-stressed barley plants. Agronomy10, 630. doi: 10.3390/agronomy10050630
75
HafezE. M.OmaraA. E. D.AlhumaydhiF. A.El-EsawiM. A. (2021). Minimizing hazard impacts of soil salinity and water stress on wheat plants by soil application of vermicompost and biochar. Physiol. Plant172, 587–602. doi: 10.1111/ppl.13261
76
HagemannN.JosephS.SchmidtH. P.KammannC. I.HarterJ.BorchT.et al. (2017). Organic coating on biochar explains its nutrient retention and stimulation of soil fertility. Nat. Commun.8, 1089. doi: 10.1038/s41467-017-01123-0
77
HaiderZ. M.HussainS.Muhammad Adnan RamzaniP.IqbalM.IqbalM.ShahzadT.et al. (2019). Bentonite and biochar mitigate Pb toxicity in Pisum sativum by reducing plant oxidative stress and Pb translocation. Plants8, 571. doi: 10.3390/plants8120571
78
HaiderG.KoyroH. W.AzamF.SteffensD.MüllerC.KammannC. (2015). Biochar but not humic acid product amendment affected maize yields via improving plant-soil moisture relations. Plant Soil.395, 141–157. doi: 10.1016/j.biortech.2019.122318
79
HaiderI.RazaM. A. S.IqbalR.AslamM. U.Habib-ur-RahmanM.RajaS.et al. (2020). Potential effects of biochar application on mitigating the drought stress implications on wheat (Triticum aestivum L.) under various growth stages. J. Saudi Chem. Soc24, 974–981. doi: 10.1016/j.jscs.2020.10.005
80
HannachiS.SignoreA.MechiL. (2023). Alleviation of associated drought and salinity stress’ detrimental impacts on an eggplant cultivar (‘Bonica F1’) by adding biochar. Plants12, 1399. doi: 10.3390/plants12061399
81
HelaouiS.BoughattasI.MkhininiM.GhazouaniH.JabnouniH.El Kribi-BoukhrisS.et al. (2023). Biochar application mitigates salt stress on maize plant: Study of the agronomic parameters, photosynthetic activities and biochemical attributes. Plant Stress9, 100182. doi: 10.1016/j.stress.2023.100182
82
HilscherA.HeisterK.SiewertC.KnickerH. (2009). Mineralisation and structural changes during the initial phase of microbial degradation of pyrogenic plant residues in soil. Org. Geochem.40, 332–342. doi: 10.1016/j.orggeochem.2008.12.004
83
HossainM. Z.BaharM. M.SarkarB.DonneS. W.OkY. S.PalansooriyaK. N.et al. (2020). Biochar and its importance on nutrient dynamics in soil and plant. Biochar2, 379–420. doi: 10.1007/s42773-020-00065-z
84
HossainM. K.StrezovV.ChanK. Y.NelsonP. F. (2010). Agronomic properties of wastewater sludge biochar and bioavailability of metals in production of cherry tomato (Lycopersicon esculentum). Chemosphere78, 1167–1171. doi: 10.1016/j.chemosphere.2010.01.009
85
HouJ.XingC.ZhangJ.WangZ.LiuM.DuanY.et al. (2024). Increase in potato yield by the combined application of biochar and organic fertilizer: key role of rhizosphere microbial diversity. Front. Plant Sci.15. doi: 10.3389/fpls.2024.1389864
86
HuangK.LiM.LiR.RasulF.ShahzadS.WuC.et al. (2023). Soil acidification and salinity: the importance of biochar application to agricultural soils. Front. Plant Sci.14. doi: 10.3389/fpls.2023.1206820
87
HuangM.ZhangZ.ZhaiY.LuP.ZhuC. (2019). Effect of straw biochar on soil properties and wheat production under saline water irrigation. Agronomy9, 457. doi: 10.3390/agronomy9080457
88
HuangJ.ZhuC.KongY.CaoX.ZhuL.ZhangY.et al. (2022). Biochar application alleviated rice salt stress via modifying soil properties and regulating soil bacterial abundance and community structure. Agronomy12, 409. doi: 10.3390/agronomy12020409
89
IbrahimH. M. E.Adam AliA. Y.ZhouG.Ibrahim ElsiddigA. M.ZhuG.Ahmed NimirN. E.et al. (2020). Biochar application affects forage sorghum under salinity stress. Chilean J. Agric. Res.80, 317–325. doi: 10.4067/S0718-58392020000300317
90
IbrahimM. E. H.AliA. Y. A.ElsiddigA. M. I.ZhouG.NimirN. E. A.AgbnaG. H.et al. (2021). Mitigation effect of biochar on sorghum seedling growth under salinity stress. Pak. J. Bot.53, 387–392. doi: 10.30848/PJB2021-2(21
91
IngraoC.MatarazzoA.GorjianS.AdamczykJ.FaillaS.PrimeranoP.et al. (2021). Wheat-straw derived bioethanol production: a review of life cycle assessments. Sci. Total Environ.781, 146751. doi: 10.1016/j.scitotenv.2021.146751
92
JabborovaD.MaH.Bellingrath-KimuraS. D.WirthS. (2021a). Impacts of biochar on basil (Ocimum basilicum) growth, root morphological traits, plant biochemical and physiological properties and soil enzymatic activities. Sci. Hortic.290, 110518. doi: 10.1016/j.scienta.2021.110518
93
JabborovaD.WirthS.HalwaniM.IbrahimM. F. M.AzabI. H. E.El-MogyM. M.et al. (2021b). Growth response of ginger (Zingiber officinale), its physiological properties and soil enzyme activities after biochar application under greenhouse conditions. Hortic7, 250. doi: 10.3390/horticulturae7080250
94
JagadeeshN.SundaramB. (2023). Adsorption of pollutants from wastewater by biochar: a review. J. Haz. Mat. Adv.9, 100226. doi: 10.1016/j.hazadv.2022.100226
95
JefferyS.VerheijenF. G.van der VeldeM.BastosA. C. (2011). A quantitative review of the effects of biochar application to soils on crop productivity using meta-analysis. Agric. Ecosyst. Environ.144, 175–187. doi: 10.1016/j.agee.2011.08.015
96
JinF.PiaoJ.MiaoS.CheW.LiX.LiX.et al. (2024). Long-term effects of biochar one-off application on soil physicochemical properties, salt concentration, nutrient availability, enzyme activity, and rice yield of highly saline-alkali paddy soils: based on a 6-year field experiment. Biochar6, 40. doi: 10.1007/s42773-024-00332-3
97
JinF.RanC.AnwariQ.GengY.GuoL.LiJ.et al. (2018). Effects of biochar on sodium ion accumulation, yield and quality of rice in saline-sodic soil of the west of Songnen plain, northeast China. Plant Soil. Environ.64, 612–618. doi: 10.17221/359/2018-PSE
98
JoteC. A. (2023). The impacts of using inorganic chemical fertilizers on the environment and human health. Org. Med. Chem. Int. J.13, 555864. doi: 10.19080/OMCIJ.2023.13.555864
99
JungS.ParkY. K.KwonE. E. (2019). Strategic use of biochar for CO2 capture and sequestration. J. CO2 Util.32, 128–139. doi: 10.1016/j.jcou.2019.04.012
100
KameyamaK.MiyamotoT.IwataY.ShionoT. (2016). Effects of biochar produced from sugarcane bagasse at different pyrolysis temperatures on water retention of a calcaric dark red soil. Soil Sci.181, 20–28. doi: 10.1097/SS.0000000000000123
101
KamranM.MalikZ.ParveenA.HuangL.RiazM.BashirS.et al. (2020). Ameliorative effects of biochar on rapeseed (Brassica napus L.) growth and heavy metal immobilization in soil irrigated with untreated wastewater. J. Plant Growth Regul.39, 266–281. doi: 10.1007/s00344-019-09980-3
102
KanwalS.IlyasN.ShabirS.SaeedM.GulR.ZahoorM.et al. (2018). Application of biochar in mitigation of negative effects of salinity stress in wheat (Triticum aestivum L.). J. Plant Nutr.41, 526–538. doi: 10.1080/01904167.2017.1392568
103
KarimiA.MoezziA.ChoromM.EnayatizamirN. (2020). Application of biochar changed the status of nutrients and biological activity in a calcareous soil. J. Soil Sci. Plant Nutr.20, 450–459. doi: 10.1007/s42729-019-00129-5
104
KaurG.AsthirB. (2017). Molecular responses to drought stress in plants. Biol. Plantarum61, 201–209. doi: 10.1007/s10535-016-0700-9
105
KhanS.IrshadS.MehmoodK.HasnainZ.NawazM.RaisA.et al. (2024). Biochar production and characteristics, its impacts on soil health, crop production, and yield enhancement: A review. Plants13, 166. doi: 10.3390/plants13020166
106
KnickerH. (2010). Black nitrogen”–an important fraction in determining the recalcitrance of charcoal. Org. Geochem41, 947–950. doi: 10.1016/j.orggeochem.2010.04.007
107
KochanekJ.LongR. L.LisleA. T.FlemattiG. R. (2016). Karrikins identified in biochars indicate post-fire chemical cues can influence community diversity and plant development. PloS One11, e0161234. doi: 10.1371/journal.pone.0161234
108
KumarD.PantK. K. (2015). Production and characterization of biocrude and biochar obtained from non-edible de-oiled seed cakes hydrothermal conversion. J. Anal. Appl. Pyrolysis115, 77–86. doi: 10.1016/j.jaap.2015.06.014
109
KumarJ. A.SathishS.PrabuD.RenitaA. A.SaravananA.DeivayanaiV. C.et al. (2023). Agricultural waste biomass for sustainable bioenergy production: Feedstock, characterization and pre-treatment methodologies. Chemosphere331, 138680. doi: 10.1016/j.chemosphere.2023.138680
110
KumarJ.SinghS.SinghM.SrivastavaP. K.MishraR. K.SinghV. P.et al. (2017). Transcriptional regulation of salinity stress in plants: A short review. Plant Gene.11, 160–169. doi: 10.1016/j.plgene.2017.04.001
111
KumariK.KhalidZ.AlamS. N.SwetaSinghB.GuldheA.et al. (2020). Biochar amendment in agricultural soil for mitigation of abiotic stress. Ecol. Pract. Appl. Sustain. Agric., 305–344. doi: 10.1007/978-981-15-3372-3_14
112
KuzyakovY.SubbotinaI.ChenH.BogomolovaI.XuX. (2009). Black carbon decomposition and incorporation into soil microbial biomass estimated by 14C labeling. Soil Biol. Biochem.41, 210–219. doi: 10.1016/j.soilbio.2008.10.016
113
LairdD.FlemingP.WangB.HortonR.KarlenD. (2010). Biochar impact on nutrient leaching from a Midwestern agricultural soil. Geoderma158, 436–442. doi: 10.1016/j.geoderma.2010.05.012
114
LairdD.NovakJ.CollinsH.IppolitoJ.KarlenD.LentzR.et al. (2017). Multi-year and multi-location soil quality and crop biomass yield responses to hardwood fast pyrolysis biochar. Geoderma289, 46–53. doi: 10.1016/j.geoderma.2016.11.025
115
LalR. (2015). Restoring soil quality to mitigate soil degradation. Sustainability7, 5875–5895. doi: 10.3390/su7055875
116
LalhriatpuiaC.TiwariD. (2023). Biochar-derived nanocomposites for environmental remediation: The insights and future perspectives. J. Environ. Chem. Eng.12, 111840. doi: 10.1016/j.jece.2023.111840
117
LangeroodiA. R. S.CampigliaE.MancinelliR.RadicettiE. (2019). Can biochar improve pumpkin productivity and its physiological characteristics under reduced irrigation regimes? Sci. Hortic.247, 195–204. doi: 10.1016/j.scienta.2018.11.059
118
LehmannJ.da SilvaJ. P.SteinerC.NehlsT.ZechW.GlaserB. (2003). Nutrient availability and leaching in an archaeological Anthrosol and a Ferralsol of the Central Amazon basin: fertilizer, manure and charcoal amendments. Plant Soil.249, 343–357. doi: 10.1023/A:1022833116184
119
LehmannJ.JosephS. (2024). “Biochar for environmental management: an introduction,” in Biochar for environmental management (London: Routledge), 1–13.
120
LehmannJ.RilligM. C.ThiesJ.MasielloC. A.HockadayW. C.CrowleyD. (2011). Biochar effects on soil biota–a review. Soil Biol. Biochem.43, 1812–1836. doi: 10.1016/j.soilbio.2011.04.022
121
LengL. J.YuanX. Z.HuangH. J.WangH.WuZ. B.FuL. H.et al. (2015). Characterization and application of bio-chars from liquefaction of microalgae, lignocellulosic biomass and sewage sludge. Fuel Process. Technol.129, 8–14. doi: 10.1016/j.fuproc.2014.08.016
122
LiY.FengH.ChenJ.LuJ.WuW.LiuX.et al. (2022b). Biochar incorporation increases winter wheat (Triticum aestivum L.) production with significantly improving soil enzyme activities at jointing stage. Catena211, 105979. doi: 10.1016/j.catena.2021.105979
123
LiD.LaiC.LiY.LiH.ChenG.LuQ. (2021b). Biochar improves cd-contaminated soil and lowers Cd accumulation in Chinese flowering cabbage (Brassica parachinensis L.). Soil Tillage Res.213, 105085. doi: 10.1016/j.still.2021.105085
124
LiJ.XuR.ZhangJ.LiC.BaoJ.LiangW. (2022a). Technical exploration of combined hydrothermal carbonization and pyrolysis to produce high-quality biochar. doi: 10.2139/ssrn.4019949. Available at SSRN 4019949.
125
LiY.YangJ.YangM.ZhangF. (2024). Exploring biochar addition impacts on soil erosion under natural rainfall: A study based on four years of field observations on the Loess Plateau. Soil Tillage Res.236, 105935. doi: 10.1016/j.still.2023.105935
126
LiL.ZhangY. J.NovakA.YangY.WangJ. (2021a). Role of biochar in improving sandy soil water retention and resilience to drought. Water13, 407. doi: 10.3390/w13040407
127
LiC.ZhangC.ZhongS.DuanJ.LiM.ShiY. (2023). The removal of pollutants from wastewater using magnetic biochar: a scientometric and visualization analysis. Molecules28, 5840. doi: 10.3390/molecules28155840
128
LiangB.LehmannJ.SolomonD.KinyangiJ.GrossmanJ.O’NeillB. J. (2006). Black carbon increases cation exchange capacity in soils. Soil Sci. Soc Am. J.70, 1719–1730. doi: 10.2136/sssaj2005.0383
129
LiuZ.DuganB.MasielloC. A.GonnermannH. M. (2017a). Biochar particle size, shape, and porosity act together to influence soil water properties. PloS One12, e0179079. doi: 10.1371/journal.pone.0179079
130
LiuA.TianD.XiangY.MoH. (2016). Effects of biochar on growth of Asian lotus (Nelumbo nucifera Gaertn.) and cadmium uptake in artificially cadmium-polluted water. Sci. Hortic.198, 311–317. doi: 10.1016/j.scienta.2015.11.030
131
LiuL.WangY.YanX.LiJ.JiaoN.HuS. (2017b). Biochar amendments increase the yield advantage of legume-based intercropping systems over monoculture. Agric. Ecosyst. Environ.237, 16–23. doi: 10.1016/j.agee.2016.12.026
132
LorenzK.LalR. (2014). Biochar application to soil for climate change mitigation by soil organic carbon sequestration. J. Plant Nutr. Soil Sci.177, 651–670. doi: 10.1002/jpln.201400058
133
MaN.ZhangL.ZhangY.YangL.YuC.YinG.et al. (2016). Biochar improves soil aggregate stability and water availability in a mollisol after three years of field application. PloS One11, e0154091. doi: 10.1371/journal.pone.0154091
134
MaharajanT.ChellasamyG.TpA. K.CeasarS. A.YunK. (2022). The role of metal transporters in phytoremediation: A closer look at Arabidopsis. Chemosphere310, 136881. doi: 10.1016/j.chemosphere.2022.136881
135
MahmoodT.KhalidS.AbdullahM.AhmedZ.ShahM. K. N.GhafoorA.et al. (2019). Insights into drought stress signaling in plants and the molecular genetic basis of cotton drought tolerance. Cells9, 105. doi: 10.3390/cells9010105
136
MandalS.PuS.AdhikariS.MaH.KimD.-H.BaiY.et al. (2020). Progress and future prospects in biochar composites: application and reflection in the soil environment. Crit. Rev. Environ. Sci. Technol51, 219–271. doi: 10.1080/10643389.2020.1713030
137
MasekO. (2022). “Biochar preparation by different thermo-chemical conversion processes,” in Eng. Biochar. Eds. SudiptaR.DineshM.OndrejM.MéndezA.TsubotaT. (Singapore: Springer), 35–46. doi: 10.1007/978-981-19-2488-0_3
138
MathankerA.DasS.PudasaineeD.KhanM.KumarA.GuptaR. (2021). A review of hydrothermal liquefaction of biomass for biofuels production with a special focus on the effect of process parameters, co-solvents, and extraction solvents. Energies14, 4916. doi: 10.3390/en14164916
139
MayaD. M. Y.LoraE. E. S.AndradeR. V.RatnerA.AngelJ. D. M. (2021). Biomass gasification using mixtures of air, saturated steam, and oxygen in a two-stage downdraft gasifier. Assessment using a CFD modeling approach. Renew. Energy.177, 1014–1030. doi: 10.1016/j.renene.2021.06.051
140
MedynskaJ. A.RivierP. A.RasseD.JonerE. J. (2020). Biochar affects heavy metal uptake in plants through interactions in the rhizosphere. Appl. Sci.10, 5105. doi: 10.3390/app10155105
141
MeenaS.ChoudharyR.SharmaS. K.ChoudharyJ.JatG.DubeyR. B.et al. (2023). Effect of lantana biochar on yield and economics of organic chickpea (Cicer arietinum L.). Pharma Innov. J.12, 2801–2803.
142
MendezA.Paz-FerreiroJ.GilE.GascóG. (2015). The effect of paper sludge and biochar addition on brown peat and coir based growing media properties. Sci. Hortic.193, 225–230. doi: 10.1016/j.scienta.2015.07.032
143
MMR (2023). Agricultural Waste Market: Market Share, Growth, and Size Projections (India: Maximize Market Research).
144
MoreiraB.CruzV. H.PérezJ. F.VianaR. (2021). Production of pellets for combustion and physisorption of CO2 from hydrothermal carbonization of food waste – Part I: High-performance solid biofuels. J. Clean. Prod.319, 128695. doi: 10.1016/j.jclepro.2021.128695
145
MukherjeeA.LalR. (2013). Biochar impacts on soil physical properties and greenhouse gas emissions. Agronomy3, 313–339. doi: 10.3390/agronomy3020313
146
MurtazaG.AhmedZ.EldinS. M.AliB.BawazeerS.UsmanM.et al. (2023). Biochar-Soil-Plant interactions: A cross talk for sustainable agriculture under changing climate. Front. Environ. Sci.11. doi: 10.3389/fenvs.2023.1059449
147
NabaviniaF.EmamiH.AstaraeeA.LakzianA. (2015). Effect of tannery wastes and biochar on soil chemical and physicochemical properties and growth traits of radish. Int. Agrophysics29, 333–339. doi: 10.1515/intag-2015-0040
148
NathH.SarkarB.MitraS.BhaladhareS. (2022). Biochar from biomass: A review on biochar preparation its modification and impact on soil including soil microbiology. Geomicrobiol. J.39, 373–388. doi: 10.1080/01490451.2022.2028942
149
NiJ.QianL.WangY.ZhangB.GuH.HuY.et al. (2022). A review on fast hydrothermal liquefaction of biomass. Fuel327, 125135. doi: 10.1016/j.fuel.2022.125135
150
NielsenS.JosephS.YeJ.ChiaC.MunroeP.van ZwietenL.et al. (2018). Crop-season and residual effects of sequentially applied mineral enhanced biochar and N fertiliser on crop yield, soil chemistry and microbial communities. Agric. Ecosyst. Environ.255, 52–61. doi: 10.1016/j.agee.2017.12.020
151
NikpourR. N.TavasoleeA.TorabianS.Farhangi-AbrizS. (2019). The effect of biochar on the physiological, morphological and anatomical characteristics of mung bean roots after exposure to salt stress. Arch. Biol. Sci.71, 321–327. doi: 10.2298/ABS190224029N
152
NourM. M.AljabiH. R.AL-HuqailA. A.HorneburgB.MohammedA. E.AlotaibiM. O. (2024). Drought responses and adaptation in plants differing in life-form. Front. Ecol. Evol.12. doi: 10.3389/fevo.2024.1452427
153
NovakJ. M.BusscherW. J.LairdD. L.AhmednaM.WattsD. W.NiandouM. A. (2009). Impact of biochar amendment on fertility of a southeastern coastal plain soil. Soil Sci.174, 105–112. doi: 10.1097/SS.0b013e3181981d9a
154
ObadiA.AlharbiA.AlomranA.AlghamdiA. G.LoukiI.AlkhashaA. (2023). Effect of biochar application on morpho-physiological traits, yield, and water use efficiency of tomato crop under water quality and drought stress. Plants12, 2355. doi: 10.3390/plants12122355
155
OguntundeP. G.AbiodunB. J.AjayiA. E.Van De GiesenN. (2008). Effects of charcoal production on soil physical properties in Ghana. J. Plant Nutr. Soil Sci.171, 591–596. doi: 10.1002/jpln.200625185
156
OkorogbonaA. O. M.ManagaL. R.AdebolaP. O.NgobeniH. M.KhosaT. B. (2015). Salinity and crop productivity. Sustain. Agricul. Rev.17, 89–120. doi: 10.1007/978-3-319-16742-8_4
157
OliverM. A.GregoryP. J. (2015). Soil, food security and human health: a review. Eur. J. Soil Sci.66, 257–276. doi: 10.1111/ejss.12216
158
OlszewskiM. P.ArauzoP. J.MaziarkaP. A.RonsseF.KruseA. (2019). Pyrolysis kinetics of hydrochars produced from Brewer’s spent grains. Catalysts9, 625. doi: 10.3390/catal9070625
159
OyebamijiY. O.AdigunB. A.ShamsudinN. A. A.IkmalA. M.SalisuM. A.MalikeF. A.et al. (2024). Recent advancements in mitigating abiotic stresses in crops. Horticulture10, 156. doi: 10.3390/horticulturae10020156
160
PanX.GuZ.ChenW.LiQ. (2021). Preparation of biochar and biochar composites and their application in a Fenton-like process for wastewater decontamination: A review. Sci. Total Environ.754, 142104. doi: 10.1016/j.scitotenv.2020.142104
161
PanditN. R.MulderJ.HaleS. E.MartinsenV.SchmidtH. P.CornelissenG. (2018). Biochar improves maize growth by alleviation of nutrient stress in a moderately acidic low-input Nepalese soil. Sci. Total Environ.625, 1380–1389. doi: 10.1016/j.scitotenv.2018.01.022
162
ParkashV.SinghS. (2020). Potential of biochar application to mitigate salinity stress in eggplant. Hortic. Sci.55, 1946–1955. doi: 10.21273/HORTSCI15398-20
163
PathyA.RayJ.ParamasivanB. (2020). Biochar amendments and its impact on soil biota for sustainable agriculture. Biochar2, 287–305. doi: 10.1007/s42773-020-00063-1
164
PaulineA. L.JosephK. (2020). Hydrothermal carbonization of organic wastes to carbonaceous solid fuel–a review of mechanisms and process parameters. Fuel27, 118472. doi: 10.1016/j.fuel.2020.118472
165
PradhanA.ChanC.RoulP. K.HalbrendtJ.SipesB. (2018). Potential of conservation agriculture (CA) for climate change adaptation and food security under rainfed uplands of India: a transdisciplinary approach. Agric. Syst.163, 27–35. doi: 10.1016/j.agsy.2017.01.002
166
PuS.LiG.TangG.ZhangY.XuW.LiP.et al. (2019). Effects of biochar on water movement characteristics in sandy soil under drip irrigation. J. Arid Land.11, 740–753. doi: 10.1007/s40333-019-0106-6
167
Pujol PereiraE. I.SuddickE. C.SixJ. (2016). Carbon abatement and emissions associated with the gasification of walnut shells for bioenergy and biochar production. PloS One11, e0150837. doi: 10.1371/journal.pone.0150837
168
PurakayasthaT. J.KumariS.PathakH. (2015). Characterisation, stability, and microbial effects of four biochars produced from crop residues. Geoderma239, 293–303. doi: 10.1016/j.geoderma.2014.11.009
169
RanC.GulaqaA.ZhuJ.WangX.ZhangS.GengY.et al. (2020). Benefits of biochar for improving ion contents, cell membrane permeability, leaf water status and yield of rice under saline–sodic paddy field condition. J. Plant Growth Reg.39, 370–377. doi: 10.1007/s00344-019-09988-9
170
RasaK.HeikkinenJ.HannulaM.ArstilaK.KuljuS.HyväluomaJ. (2018). How and why does willow biochar increase a clay soil water retention capacity? Biomass Bioenergy119, 346–353. doi: 10.1016/j.biombioe.2018.10.004
171
RavichandranS. R.VenkatachalamC. D.SengottianM.SekarS.KandasamyS.SubramanianK. P.et al. (2022). A review on hydrothermal liquefaction of algal biomass on process parameters, purification and applications. Fuel313, 122679. doi: 10.1016/j.fuel.2021.122679
172
RazzaghiF.ObourP. B.ArthurE. (2020). Does biochar improve soil water retention? A systematic review and meta-analysis. Geoderma361, 114055. doi: 10.1016/j.geoderma.2019.114055
173
RogovskaN.LairdD. A.KarlenD. L. (2016). Corn and soil response to biochar application and stover harvest. Field Crops Res.187, 96–106. doi: 10.1016/j.fcr.2015.12.013
174
RuggieroA.PunzoP.LandiS.CostaA.Van OostenM. J.GrilloS. (2017). Improving plant water use efficiency through molecular genetics. Hortic. Sci.3, 31. doi: 10.3390/horticulturae3020031
175
SakhiyaA. K.AnandA.KaushalP. (2020). Production, activation, and applications of biochar in recent times. Biochar2, 253–285. doi: 10.1007/s42773-020-00047-1
176
SaqibN. U.SharmaH. B.BaroutianS.DubeyB.SarmahA. K. (2019). Valorisation of food waste via hydrothermal carbonisation and techno-economic feasibility assessment. Sci. Total Environ.690, 261–276. doi: 10.1016/j.scitotenv.2019.06.484
177
SasakiC.OkumuraR.AsadaC.NakamuraY. (2014). Steam explosion treatment for ethanol production from branches pruned from pear trees by simultaneous saccharification and fermentation. Biosci. Biotechnol. Biochem.78, 160–166. doi: 10.1080/09168451.2014.877818
178
SattarA.SherA.IjazM.Ul-AllahS.ButtM.IrfanM.et al. (2020). Interactive effect of biochar and silicon on improving morpho-physiological and biochemical attributes of maize by reducing drought hazards. J. Soil Sci. Plant Nutr.20, 1819–1826. doi: 10.1007/s42729-020-00253-7
179
SawargaonkarG.PasumarthiR.KaleS.ChoudhariP.RakeshS.MutnuriS.et al. (2024). Valorization of peanut shells through biochar production using slow and fast pyrolysis and its detailed physicochemical characterization. Front. Sustain.5. doi: 10.3389/frsus.2024.1417207
180
ShahbazA. K.LewińskaK.IqbalJ.AliQ.IqbalM.AbbasF.et al. (2018). Improvement in productivity, nutritional quality, and antioxidative defense mechanisms of sunflower (Helianthus annuus L.) and maize (Zea mays L.) in nickel contaminated soil amended with different biochar and zeolite ratios. J. Environ. Manage.218, 256–270. doi: 10.1016/j.jenvman.2018.04.046
181
SheD.SunX.GamareldawlaA. H.NazarE. A.HuW.EdithK.et al. (2018). Benefits of soil biochar amendments to tomato growth under saline water irrigation. Sci. Rep.8, 14743. doi: 10.1038/s41598-018-33040-7
182
ShenX.HuangD. Y.RenX. F.ZhuH. H.WangS.XuC.et al. (2016). Phytoavailability of Cd and Pb in crop straw biochar-amended soil is related to the heavy metal content of both biochar and soil. J. Environ. Manage.168, 245–251. doi: 10.1016/j.jenvman.2015.12.019
183
SinghB. P.CowieA. L. (2014). Long-term influence of biochar on native organic carbon mineralization in a low-carbon clayey soil. Sci. Rep.4, 3687. doi: 10.1038/srep03687
184
SinghH.NorthupB. K.RiceC. W.PrasadP. V. (2022). Biochar applications influence soil physical and chemical properties, microbial diversity, and crop productivity: a meta-analysis. Biochar4, 8. doi: 10.1007/s42773-022-00138-1
185
SivaranjaneeR.KumarP. S.ChitraB.RangasamyG. (2024). A critical review on biochar for the removal of toxic pollutants from water environment. Chemos360, 142382. doi: 10.1016/j.chemosphere.2024.142382
186
SiwalS. S.ZhangQ.SunC.ThakurS.GuptaV. K.ThakurV. K. (2020). Energy production from steam gasification processes and parameters that contemplate in biomass gasifier a review. Bioresour. Technol.297, 122481. doi: 10.1016/j.biortech.2019.122481
187
SousaA. A. T. C.FigueiredoC. (2016). Sewage sludge biochar: effects on soil fertility and growth of radish. Biol. Agric. Hortic.32, 127–138. doi: 10.1080/01448765.2015.1093545
188
SteinerC.TeixeiraW. G.LehmannJ.NehlsT.de MacêdoJ. L. V.BlumW. E.et al. (2007). Long term effects of manure, charcoal and mineral fertilization on crop production and fertility on a highly weathered Central Amazonian upland soil. Plant Soil.291, 275–290. doi: 10.1007/s11104-007-9193-9
189
SunJ.FanQ.MaJ.CuiL.QuanG.YanJ.et al. (2020). Effects of biochar on cadmium (Cd) uptake in vegetables and its natural downward movement in saline-alkali soil. Environ. pollut. Bioavailab.32, 36–46. doi: 10.1080/26395940.2020.1714487
190
SunF.LuS. (2014). Biochars improve aggregate stability, water retention, and pore-space properties of clayey soil. J. Plant Nutr. Soil Sci.177, 26–33. doi: 10.1002/jpln.201200639
191
TahirS.GulS.Aslam GhoriS.SohailM.BatoolS.JamilN.et al. (2018). Biochar influences growth performance and heavy metal accumulation in spinach under wastewater irrigation. Cogent. Food. Agric.4, 1467253. doi: 10.1080/23311932.2018.1467253
192
TanM. (2023). Conversion of agricultural biomass into valuable biochar and their competence on soil fertility enrichment. Environ. Res.234, 116596. doi: 10.1016/j.envres.2023.116596
193
ThinesK.AbdullahE.MubarakN.RuthiraanM. (2017). Synthesis of magnetic biochar from agricultural waste biomass to enhancing route for wastewater and polymer application: a review. Renew. Sust. Energy Rev.67, 257–276. doi: 10.1016/j.rser.2016.09.057
194
TomczykA.SokołowskaZ.BogutaP. (2020). Biochar physicochemical properties: pyrolysis temperature and feedstock kind effects. Rev. Environ. Sci. Biotechnol.19, 191–215. doi: 10.1007/s11157-020-09523-3
195
Van DijkM.MorleyT.RauM. L.SaghaiY. (2021). A meta-analysis of projected global food demand and population at risk of hunger for the period 2010–2050. Nat. Food.2, 494–501. doi: 10.1038/s43016-021-00322-9
196
VerheijenF. G.ZhuravelA.SilvaF. C.AmaroA.Ben-HurM.KeizerJ. J. (2019). The influence of biochar particle size and concentration on bulk density and maximum water holding capacity of sandy vs sandy loam soil in a column experiment. Geoderma347, 194–202. doi: 10.1016/j.geoderma.2019.03.044
197
WanQ.YuanJ. H.XuR. K.LiX. H. (2014). Pyrolysis temperature influences ameliorating effects of biochars on acidic soil. Environ. Sci. pollut. Res.21, 2486–2495. doi: 10.1007/s11356-013-2183-y
198
WangG.DaiY.YangH.XiongQ.WangK.ZhouJ.et al. (2020a). A review of recent advances in biomass pyrolysis. Energy Fuel.34, 15557–15578. doi: 10.1021/acs.energyfuels.0c03107
199
WangD.JiangP.ZhangH.YuanW. (2020b). Biochar production and applications in agro and forestry systems: A review. Sci. Total Environ.723, 137775. doi: 10.1016/j.scitotenv.2020.137775
200
WangY.MaZ.WangX.SunQ.DongH.WangG.et al. (2019). Effects of biochar on the growth of apple seedlings, soil enzyme activities and fungal communities in replant disease soil. Sci. Hortic.256, 108641. doi: 10.1016/j.scienta.2019.108641
201
WangJ.XiongZ.KuzyakovY. (2016). Biochar stability in soil: meta-analysis of decomposition and priming effects. GCB Bioenergy8, 512–523. doi: 10.1111/gcbb.12266
202
WangS.ZhengJ.WangY.YangQ.ChenT.ChenY.et al. (2021). Photosynthesis, chlorophyll fluorescence, and yield of peanut in response to biochar application. Front. Plant Sci.12. doi: 10.3389/fpls.2021.650432
203
WaniO. A.ParthibanM.BhatM. A.MahdiS. S.JanR.BhatM. A.et al. (2022). “Biochar: A new emerging tool to mitigate abiotic stresses and its effect on soil properties,” in Secondary Agriculture. Eds. BaharF. A.Anwar BhatM.MahdiS. S. (Springer, Cham). doi: 10.1007/978-3-031-09218-3_9
204
WeiJ.TuC.YuanG.LiuY.BiD.XiaoL.et al. (2019). Assessing the effect of pyrolysis temperature on the molecular properties and copper sorption capacity of a halophyte biochar. Environ. pollut.251, 56–65. doi: 10.1016/j.envpol.2019.04.128
205
WenZ.ChenY.LiuZ.MengJ. (2022). Biochar and Arbuscular mycorrhizal fungi stimulate rice root growth strategy and soil nutrient availability. Eur. J. Soil Biol.113, 103448. doi: 10.1016/j.ejsobi.2022.103448
206
WiednerK.NaisseC.RumpelC.PozziA.WieczorekP.GlaserB. (2013). Chemical modification of biomass residues during hydrothermal carbonization–What makes the difference, temperature or feedstock? Org. Geochem54, 91–100. doi: 10.1016/j.orggeochem.2012.10.006
207
WindeattJ. H.RossA. B.WilliamsP. T.ForsterP. M.NahilM. A.SinghS. (2014). Characteristics of biochars from crop residues: Potential for carbon sequestration and soil amendment. J. Environ. Manage.146, 189–197. doi: 10.1016/j.jenvman.2014.08.003
208
WoldetsadikD.DrechselP.KeraitaB.MarschnerB.ItannaF.GebrekidanH. (2016). Effects of biochar and alkaline amendments on cadmium immobilization, selected nutrient and cadmium concentrations of lettuce (Lactuca sativa) in two contrasting soils. Springer Plus.5, 1–16. doi: 10.1186/s40064-016-2019-6
209
WuJ.JinL.WangN.WeiD.PangM.LiD.et al. (2023). Effects of combined application of chemical fertilizer and biochar on soil physio-biochemical properties and maize. Yield. Agric.13, 1200. doi: 10.3390/agriculture13061200
210
WuW.YangM.FengQ.McGroutherK.WangH.LuH.et al. (2012). Chemical characterization of rice straw-derived biochar for soil amendment. Biomass. Bioenergy47, 268–276. doi: 10.1016/j.biombioe.2012.09.034
211
XiaoQ.ZhuL. X.ZhangH. P.LiX. Y.ShenY. F.LiS. Q. (2016). Soil amendment with biochar increases maize yields in a semi-arid region by improving soil quality and root growth. Crop Pasture. Sci.67, 495–507. doi: 10.1071/CP15351
212
XuH. J.WangX. H.LiH.YaoH. Y.SuJ. Q.ZhuY. G. (2014). Biochar impacts soil microbial community composition and nitrogen cycling in an acidic soil planted with rape. Environ. Sci. Technol.48, 9391–9399. doi: 10.1021/es502105
213
YaashikaaP. R.KumarP. S.VarjaniS.SaravananA. (2020). A critical review on the biochar production techniques, characterization, stability and applications for circular bioeconomy. Biotechnol. Rep.28, e00570. doi: 10.1016/j.btre.2020.e00570
214
YangA.AkhtarS. S.LiL.FuQ.LiQ.NaeemM. A.et al. (2020). Biochar mitigates combined effects of drought and salinity stress in quinoa. Agronomy10, 912. doi: 10.3390/agronomy10060912
215
YaoQ.LiuJ.YuZ.LiY.JinJ.LiuX.et al. (2017). Three years of biochar amendment alters soil physiochemical properties and fungal community composition in a black soil of Northeast China. Soil Biol. Biochem.110, 56–67. doi: 10.1016/j.soilbio.2017.03.005
216
YasmeenS.WahabA.SaleemM. H.AliB.QureshiK. A.JaremkoM. (2022). Melatonin as a foliar application and adaptation in lentil (Lens culinaris medik.) crops under drought stress. Sustain14, 16345. doi: 10.3390/su142416345
217
YildirimE.EkinciM.TuranM. (2021). Impact of biochar in mitigating the negative effect of drought stress on cabbage seedlings. J. Soil Sci. Plant Nutr.21, 2297–2309. doi: 10.1007/s42729-021-00522-z
218
YouS.OkY. S.TsangD. C.KwonE. E.WangC. H. (2018). Towards practical application of gasification: a critical review from syngas and biochar perspectives. Crit. Rev. Environ. Sci. Technol.48, 1165–1213. doi: 10.1080/10643389.2018.1518860
219
YounisU.MalikS. A.RizwanM.QayyumM. F.OkY. S.ShahM. H. R.et al. (2016). Biochar enhances the cadmium tolerance in spinach (Spinacia oleracea) through modification of Cd uptake and physiological and biochemical attributes. Environ. Sci. pollut. Res.23, 21385–21394. doi: 10.1007/s11356-016-7344-3
220
YounisA.RamzanF.RamzanY.ZulfiqarF.AhsanM.LimK. B. (2020). Molecular markers improve abiotic stress tolerance in crops: a review. Plants9, 1374. doi: 10.3390/plants9101374
221
Zafar-ul-HyeM.Tahzeeb-ul-HassanM.MuhammadA.FahadS.MartinB.TerezaD.et al. (2020). Potential role of compost mixed biochar with rhizobacteria in mitigating lead toxicity in spinach. Sci. Rep.10, 12159. doi: 10.1038/s41598-020-69183-9
222
ZaheerM. S.AliH. H.SoufanW.IqbalR.Habib-ur-RahmanM.IqbalJ.et al. (2021). Potential effects of biochar application for improving wheat (Triticum aestivum L.) growth and soil biochemical properties under drought stress conditions. Land10, 1125. doi: 10.3390/land10111125
223
ZhangJ.BaiZ.HuangJ.HussainS.ZhaoF.ZhuC.et al. (2019). Biochar alleviated the salt stress of induced saline paddy soil and improved the biochemical characteristics of rice seedlings differing in salt tolerance. Soil Tillage Res.195, 104372. doi: 10.1016/j.still.2019.104372
224
ZhangA.BianR.PanG.CuiL.HussainQ.LiL. (2012a). Effects of biochar amendment on soil quality, crop yield and greenhouse gas emission in a Chinese rice paddy: a field study of 2 consecutive rice growing cycles. Field Crops Res.127, 153–160. doi: 10.1016/j.fcr.2011.11.020
225
ZhangW.ChenJ.FangH.ZhangG.ZhuZ.XuW.et al. (2022). Simulation on cogasification of bituminous coal and industrial sludge in a downdraft fixed bed gasifier coupling with sensible heat recovery, and potential application in sludge-to-energy. Energy243, 123052. doi: 10.1016/j.energy.2021.123052
226
ZhangY.DingJ.WangH.SuL.ZhaoC. (2020b). Biochar addition alleviates the negative effects of drought and salinity stress on soybean productivity and water use efficiency. BMC Plant Biol.20, 1–11. doi: 10.1186/s12870-020-02493-2
227
ZhangM.GaoB.YaoY.XueY.InyangM. (2012b). Synthesis of porous MgO-biochar nanocomposites for removal of phosphate and nitrate from aqueous solutions. Chem. Eng. J.210, 26–32. doi: 10.1016/j.cej.2012.08.052
228
ZhangQ. Q.SongY. F.WuZ.YanX. Y.GuninaA.KuzyakovY.et al. (2020a). Effects of six-year biochar amendment on soil aggregation, crop growth, and nitrogen and phosphorus use efficiencies in a rice-wheat rotation. J. Clean. Prod.242, 118435. doi: 10.1016/j.jclepro.2019.118435
229
ZhangY.WangJ.FengY. (2021). The effects of biochar addition on soil physicochemical properties: A review. Catena202, 105284. doi: 10.1016/j.catena.2021.105284
230
ZhangS.WangL.GaoJ.ZhouB.HaoW.FengD.et al. (2024). Effect of biochar on biochemical properties of saline soil and growth of rice. Heliyon10, e23859. doi: 10.1016/j.heliyon.2023.e23859
231
ZhangX.WangH.HeL.LuK.SarmahA.LiJ.et al. (2013). Using biochar for remediation of soils contaminated with heavy metals and organic pollutants. Environ. Sci. pollut. Res.20, 8472–8483. doi: 10.1007/s11356-013-1659-0
232
ZhangW.WeiJ.GuoL.FangH.LiuX.LiangK.et al. (2023). Effects of two biochar types on mitigating drought and salt stress in tomato seedlings. Agronomy13, 1039. doi: 10.3390/agronomy13041039
233
ZouZ.MiW.LiX.HuQ.ZhangL.ZhangL.et al. (2023). Biochar application method influences root growth of tea (Camellia sinensis L.) by altering soil biochemical properties. Sci. Hortic.315, 111960. doi: 10.1016/j.scienta.2023.111960
234
ZulfiqarB.RazaM. A. S.SaleemM. F.AslamM. U.IqbalR.MuhammadF.et al. (2022). Biochar enhances wheat crop productivity by mitigating the effects of drought: Insights into physiological and antioxidant defense mechanisms. PloS One17, e0. doi: 10.1371/journal.pone.0276350
Summary
Keywords
abiotic stress, biochar (BC), BC synthesis, crop improvement, soil properties, soil stress alleviation
Citation
Rathinapriya P, Maharajan T, Jothi R, Prabakaran M, Lee I-B, Yi P-H and Jeong ST (2025) Unlocking biochar impacts on abiotic stress dynamics: a systematic review of soil quality and crop improvement. Front. Plant Sci. 15:1479925. doi: 10.3389/fpls.2024.1479925
Received
13 August 2024
Accepted
20 December 2024
Published
13 January 2025
Volume
15 - 2024
Edited by
Rabia Nazir, Pakistan Council of Scientific & Industrial Research, Pakistan
Reviewed by
Alio Moussa Abdourazak, Abdou Moumouni University of Niamey, Niger
Romina Alina Marc, University of Agricultural Sciences and Veterinary Medicine Cluj-Napoca, Romania
Mjv Largia, St.Xavier’s College, India
Updates
Copyright
© 2025 Rathinapriya, Maharajan, Jothi, Prabakaran, Lee, Yi and Jeong.
This is an open-access article distributed under the terms of the Creative Commons Attribution License (CC BY). The use, distribution or reproduction in other forums is permitted, provided the original author(s) and the copyright owner(s) are credited and that the original publication in this journal is cited, in accordance with accepted academic practice. No use, distribution or reproduction is permitted which does not comply with these terms.
*Correspondence: Seung Tak Jeong, jst0ry@korea.kr
Disclaimer
All claims expressed in this article are solely those of the authors and do not necessarily represent those of their affiliated organizations, or those of the publisher, the editors and the reviewers. Any product that may be evaluated in this article or claim that may be made by its manufacturer is not guaranteed or endorsed by the publisher.